
Although social deterioration in drug addiction has been widely acknowledged clinically, little is known about altered social interactive patterns and their intra- and inter-brain neural underpinnings. The in-depth investigation into the behavioral and neural mechanisms underlying how individuals with heroin use disorder (HUD) engage in cooperation and competition—two fundamental forms of social interaction—is crucial for comprehensively characterizing atypical social interaction in HUD. We utilized functional near-infrared spectroscopy (fNIRS) hyperscanning to explore the cooperative and competitive patterns in individuals with HUD during a real-time interactive task. Compared to healthy control dyads, HUD dyads exhibited a higher error rate under both cooperative and competitive conditions. HUD participants showed reduced inter-brain synchronization (IBS) in the prefrontal cortex (PFC) and right temporoparietal junction (r-TPJ), as well as decreased PFC activation during cooperation compared to healthy controls. In contrast, both IBS and PFC activity were higher during competition than during cooperation. Critically, IBS in the r-TPJ mediated the relationship between heroin craving and cooperative performance, suggesting a potential target for neurofeedback interventions. These findings reveal impaired cooperative abilities and heightened competitive tendencies in HUD, offering translational insights for the development of targeted interventions.
Heroin use disorder (HUD) constitutes a major global health concern, affecting an estimated 30 million individuals—approximately 0.6% of the worldwide population (Volkow & Blanco, 2021). Characterized by persistent and compulsive drug-seeking behavior, HUD profoundly disrupts not only physical health but also psychosocial functioning (Hasin et al., 2012; Verdejo-Garcia, 2014). Social dysfunction associated with HUD undermines treatment adherence, thereby exacerbating cravings and increasing the risk of relapse (Chan et al., 2019; Rawas et al., 2020; Volkow & Boyle, 2018). Despite this clinical relevance, the aberrant patterns of social interaction in individuals with HUD and underlying neural correlates remain poorly understood in real-world social contexts.
Social interaction plays a critical role in building and sustaining interpersonal relationships (Holt‐Lunstad, 2024), yet drug use severely impairs this fundamental aspect of human behavior. Aberrant social interaction is a hallmark of numerous psychiatric disorders and precipitates overt interpersonal and societal difficulties (Schilbach, 2016; Wei et al., 2023). Acute heroin use, as a prototypical opioid exposure, induces a transient sense of social connectedness that diminishes motivation to pursue authentic interpersonal interactions (Christie, 2021). Over time, this diminished motivation progressively contracts social networks and exacerbates social withdrawal (Christie, 2021). Successful cooperation requires coordinated interaction with partners to achieve shared goals (Lu et al., 2025). However, reduced social engagement can disrupt the typical dynamics of cooperation. Chronic heroin use downregulates sensitivity to natural rewards from social behavior, and the consequent experience of social isolation will drive increasing craving for drug-induced euphoria.
Cooperation and competition represent two fundamental forms of social interaction prevalent across diverse social relationships (Johnson, 2003). While these two dynamics are inherently opposing, they are also closely interrelated. By pursuing personal goals through impeding or undermining the efforts of others, competition often disrupts the formation and maintenance of interdependent interpersonal relationships (Liu et al., 2024). While cooperative deficits in addiction have been studied, the competitive dimension—potentially reflecting maladaptive compensation—remains unexplored. Chronic drug users are typically characterized by impaired self-control and diminished moral judgment. They often display heightened aggression and risk-taking behaviour, alongside reduced prosocial behaviour (Blanco-Gandía et al., 2015; Zacher et al., 2024). Concurrently investigating both cooperative and competitive interactions could reveal HUD-specific social motivation imbalances and provide a comprehensive characterisation of aberrant social interaction in this population.
Most existing studies examine these social deficits from a single-brain perspective, which ignores the fact that social behavior involves complex and dynamic interpersonal coordination processes between individuals (Schilbach & Redcay, 2025). To gain a deeper understanding of social dysfunction in HUD, it is essential to adopt a naturalistic real-time interaction paradigm to assess the aberrant interpersonal interaction patterns, as well as their intra-brain and inter-brain neural signatures. fNIRS-based hyperscanning is a powerful tool for investigating real-time social interaction patterns (Balconi & Vanutelli, 2017b), yet its application to unveil novel neural mechanisms underlying social dysfunction in addiction remains overlooked (Carollo et al., 2022).
The prefrontal cortex (PFC) and the right temporoparietal junction (r-TPJ) are critically involved in social interactions, as demonstrated by neuroimaging studies examining inter-brain synchrony (IBS) and brain activation levels (Konovalov, 2021; Li et al., 2018). Increased craving for drugs is associated with more blunted responses to genuine social rewards, indicating severe neuroadaptive alterations (Venniro et al., 2019, 2022). Chronic opioid addiction has been associated with structural and functional abnormalities in the PFC and r-TPJ, potentially resulting from drug-induced neurotoxicity (Ceceli et al., 2022; Luo et al., 2020; Pandria et al., 2018). These disruptions are thought to impair the processing of social rewards and hinder effective social coordination.
According to the coordination-synchrony hypothesis, deficits in coordination ability lead to reduced IBS in individuals with neurological damage (Bilek et al., 2017; Wei et al., 2023). Additionally, insensitivity to social rewards and neurological impairments are also reflected in insufficient activation levels in the brain (Liu et al., 2023). Exploring these potential neural abnormalities during interactive processes is crucial for comprehending the pathological basis of social functional deficits in drug addiction and for developing neuroregulatory interventions targeting precise biological markers.
Furthermore, while prior research has primarily focused on cooperative interactions, recent experiments in rats have indicated that social competition may contribute to addiction treatment (Deng et al., 2025). However, the neural signatures evoked by social competitive interactions in humans with HUD remain unknown, leaving an important research gap. Because competition involves perceiving and understanding others’ intentions, it typically elicits a similar but lower IBS than cooperation (Lei et al., 2025; Liu et al., 2017; Zhang et al., 2023). This neural pattern may differ in individuals with HUD. As noted earlier, they may display heightened competitiveness and a greater willingness to allocate cognitive resources toward understanding, imitating, and predicting the behaviour of others under the competitive condition. Such increased investment and hyper-mentalizing may result in excessively elevated IBS during competition (Alon et al., 2024). Moreover, since competitive behaviour also relies on neural activity within regions such as the PFC and r-TPJ (Zhang et al., 2023), and individuals with HUD may demonstrate a stronger tendency toward competitive engagement, they are likely to show enhanced neural activation in these areas during competitive tasks.
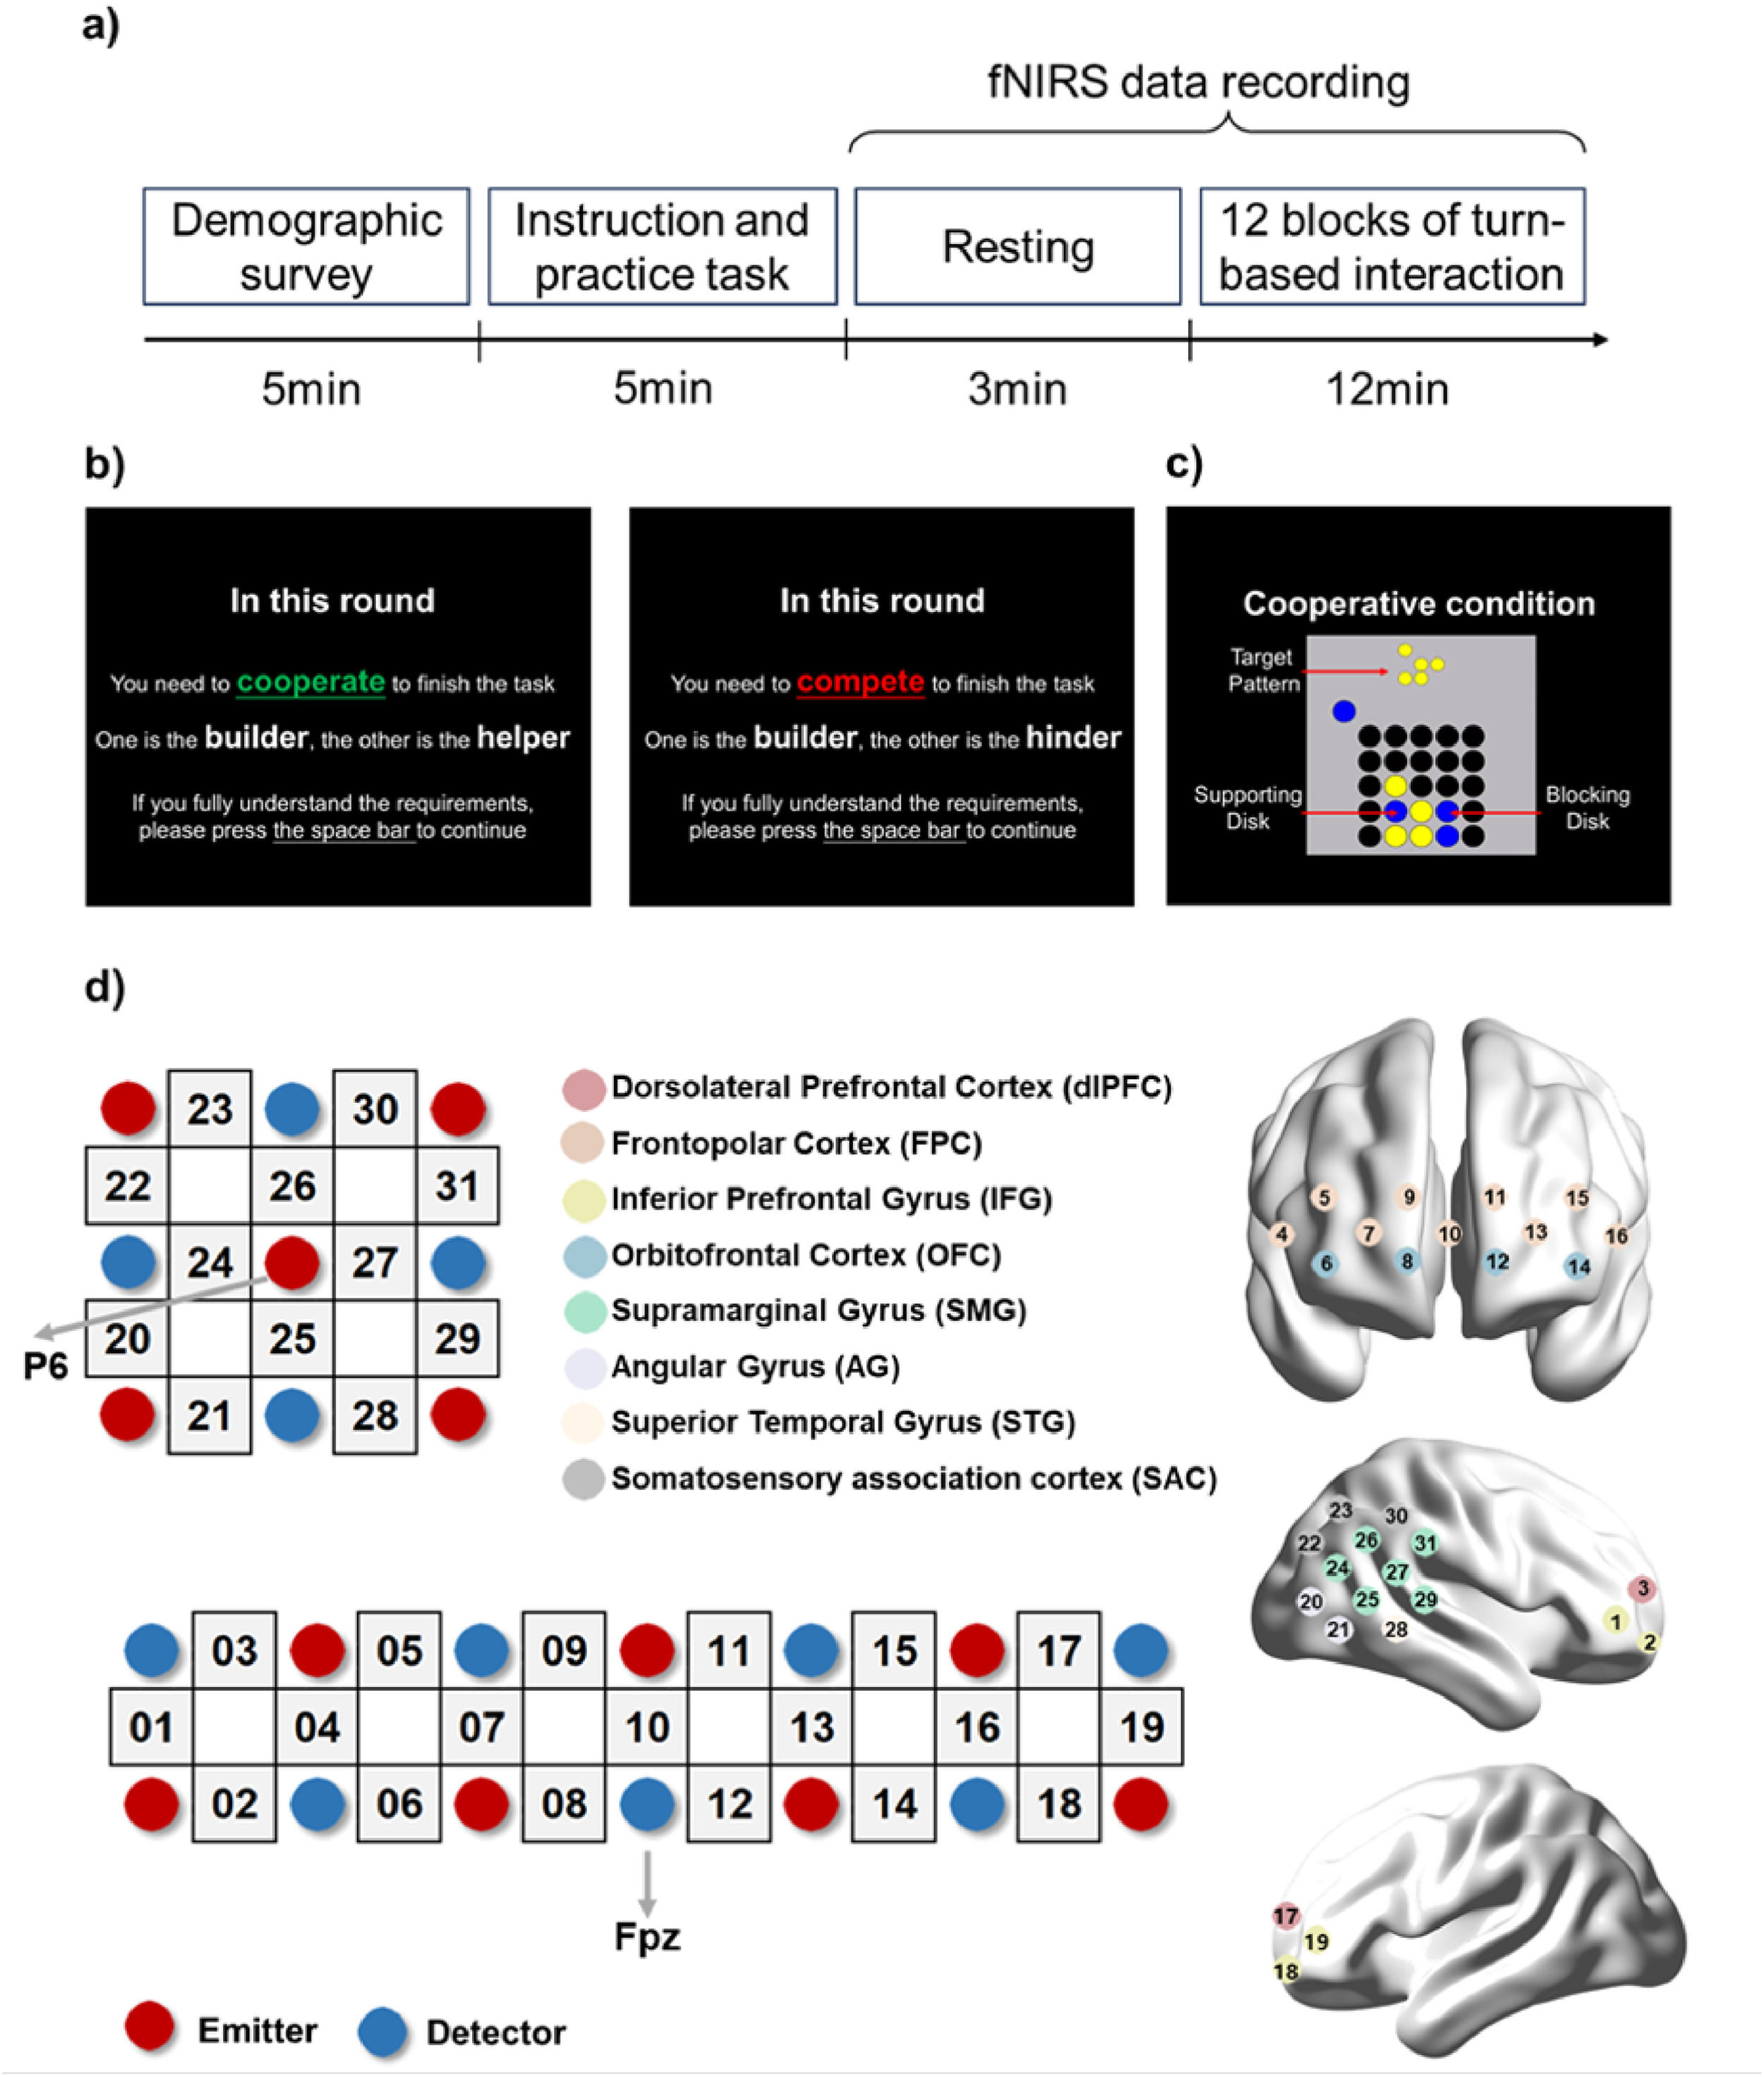
The current research aimed to investigate atypical social interactive patterns and their neural correlates both within individual brains and across interacting brains in individuals with HUD. A turn-based Pattern Game paradigm was employed to elicit dyadic real-time interactions in both cooperative and competitive contexts (Fig. 1a–c). Neural responses in the PFC and r-TPJ were simultaneously recorded using fNIRS (Fig. 1d). Building on prior findings, we proposed the following hypotheses: (1) Individuals with HUD would demonstrate abnormal behavioural patterns under the cooperative or competitive condition relative to healthy controls; (2) During cooperation, individuals with HUD would exhibit reduced IBS and lower individual brain activation in the PFC and r-TPJ, whereas during competition, they would show increased IBS and heightened activation in these regions; (3) since the IBS may serve as a potential biomarker linking clinical symptoms and task performance, IBS under the cooperative condition in individuals with HUD would mediate the relationship between addiction-related symptoms and behavioural deficits.
Materials and methodsParticipants
Recruitment of participants with HUD was conducted in two drug rehabilitation centres in Shaanxi Province, China. A group of HC participants was also recruited and matched to the HUD participants in terms of age, gender, and educational attainment. The inclusion criteria for the HUD group were as follows: 1) HUD matched the diagnostic criteria for opioid use disorder (OUD) outlined in the Fifth Edition of the Diagnostic and Statistical Manual of Mental Disorders (DSM-5); 2) each participant with HUD consumed an average of 0.1 grams or more of heroin per day, with positive heroin urine tests before entering the rehabilitation; 3) all participants had no current or past diagnoses of mental illness. To control for the potential confounding effects of treatment-related variables, all the HUD participants underwent a uniform detoxification rehabilitation program without medication-assisted treatment, had no history of polysubstance use, and were in the acute detoxification rehabilitation phase. These characteristics have been described to clarify the control of extraneous variables for the clinical sample.
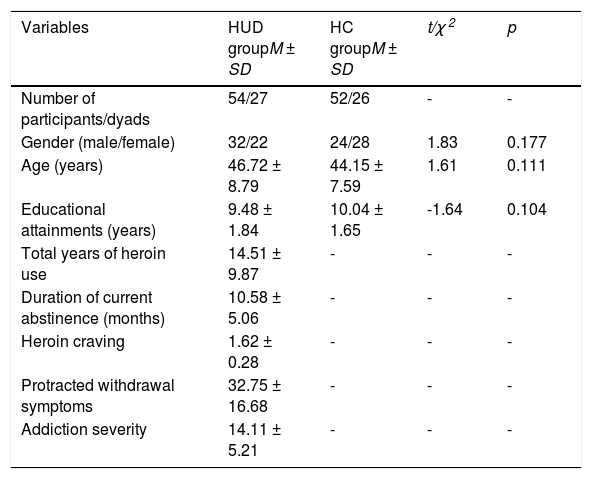
The differences in demographic information between the HUD and HC groups were not significant. Table 1 presents detailed demographic and clinical characteristics. All participants provided written informed consent indicating their understanding of the study procedures prior to participation. They received monetary compensation upon completion of the entire experiment. This study was in accordance with the ethical principles outlined in the Helsinki Declaration and received approval from the Academic Committee of Key Laboratory of Modern Teaching Technology, Ministry of Education, Shaanxi Normal University in China (No. L20231117-03).
Demographic information of participants.
Note: HUD: heroin use disorder, HC: healthy control.
HUD participants and HC participants were separately randomly paired in dyads, forming 27 HUD dyads and 26 HC dyads. Consistent with previous studies, dyads were formed with two same-sex strangers to exclude the potential effect of gender and familiarity (Zhao et al., 2022, 2023). Based on our experimental design, a priori power analysis using G*Power 3.1.9.7 suggested that a total of 46 dyads would be necessary to detect a medium effect size (Cohen's f = 0.25) with Type Ⅰ error of 0.05 (α = 0.05) and Type Ⅱ error of 0.10 (1 - β = 0.90), confirming our sample size was adequate (Faul et al., 2007).
Tasks and proceduresAddiction-related IndicatorsThree questionnaires were used to measure the heroin addiction-related indicators of the participants with HUD.
The Heroin Craving Questionnaire (HCQ) was employed to measure heroin craving intensity (Liu et al., 2006). This scale comprised 25 items. Each item was rated on a 7-point Likert scale from 1 (never) to 7 (always), with reverse scoring applied to specific items marked with an asterisk. The mean score across all items was calculated to standardize the measurement, with higher scores indicating more severe craving symptoms.
The Protracted Withdrawal Symptoms (PWS) was utilized to evaluate withdrawal symptoms (Liu et al., 2000). This 19-item scale assessed symptoms across four domains, with each item rated from 0 (no symptoms) to 4 (extremely severe symptoms). The total score, calculated by summing all item scores, reflected the overall severity of protracted withdrawal symptoms, with higher scores indicating more severe withdrawal experiences.
The Opioid Addiction Severity Inventory (OASI) was administered to assess the severity of opioid addiction (Lian & Liu, 2004). This 12-item scale evaluated various symptoms using a 4-point rating scale: 0 (no symptoms), 1 (mild symptoms), 2 (moderate symptoms), and 3 (severe symptoms). The total score, ranging from 0 to 36, was calculated by summing all item scores, with higher scores indicating more severe addiction.
Experimental design and procedureThe turn-based interactive Pattern Game paradigm was used to investigate the social interaction performance in cooperative and competitive contexts (Liu et al., 2017; Zhao et al., 2022). Two participants sat adjacent to a shared computer display. They were instructed on the rules and operational requirements of the experimental task. A video was presented to more clearly visualize the task procedure. After confirming that participants fully understood the task, the practice task with one round of each condition was performed. Subsequently, the formal task was conducted after 3 minutes of collection of fNIRS rest-state baseline data. In the baseline acquisition, participants closed their eyes and remained relaxed. The whole formal task lasted for approximately 12 minutes. fNIRS data were recorded throughout the whole task (Fig. 1a).
Pattern GameThe Pattern Game task consisted of three conditions: the cooperative condition, the competitive condition, and the independent condition (Liu et al., 2017; Zhao et al., 2022) (Fig. 1b). One of the participants acted as the builder, and the other one acted as the helper in the cooperation condition, the hinderer in the competition condition, or the observer in the independent condition. The experiment comprised 12 blocks, with four blocks per condition, and each block contained two trials. This paradigm has been validated in several studies on interpersonal interaction for its effectiveness in differentiating between cooperative and competitive contexts through standardized instructions and task settings (Liu et al., 2017; Zhao et al., 2022).
Before the formal task, all participants thoroughly understood the cooperative and competitive contexts and the corresponding role rules through standardized video tutorials and practice sessions. The tutorial explicitly stated that in the cooperative condition, the helper should assist the builder in completing the target pattern, and in the competitive condition, the hinderer should disrupt the builder from matching the target pattern by occupying the wrong position or placing disks incorrectly. Before each block, participants were presented with a dedicated instruction screen that clearly stated the interpersonal goal for the upcoming block. In the cooperative condition, they were explicitly instructed: "You and your partner are in a cooperative relationship, and you need to help him/her complete this diagram"; in the competitive condition, they were explicitly instructed: "You and your partner are in a competitive relationship, and you need to hinder him/her from completing the pattern." The screen prominently displayed the condition name (e.g., "cooperate" in bold font) and explicitly described the role requirements. Participants were required to press the space bar to confirm their understanding before the block began. To ensure comprehension, all participants completed practice sessions prior to the formal task. During the practice, the experimenter observed in real-time and confirmed that participants' behaviors complied with the role rules, ensuring they correctly adopted the intended interpersonal goals.
A 5 × 5 matrix board appeared in the task interface, with a target pattern consisting of 5 disks on top of the board (Fig. 1c). The two participants took turns moving disks to build the pattern in the empty slot together. The goal of the builder was to reproduce the target pattern. In the cooperative condition, the helper needed to assist the builder in completing the construction of the target pattern. In contrast, in the competitive condition, the hinderer disrupted the builder's alignment of the target pattern by either occupying the position of the target pattern or by putting the disk in the wrong position. In the independent condition, the builder was solely responsible for the construction of the target pattern, with the observer watching.
The order of the three conditions (cooperative, competitive, independent) was fully randomized across the experiment. Additionally, within each condition, the assignment of roles (e.g., builder vs. helper in the cooperative condition; builder vs. hinderer in the competitive condition) was counterbalanced across blocks. This fully randomized and counterbalanced design effectively controls for potential confounds arising from practice effects, fatigue, and order effects, ensuring that the observed effects are primarily attributable to the manipulation of the social context. To further minimize inferences between the different blocks, a gaze point "+" was presented lasting for 15 seconds before the start of each block, allowing oxyhemoglobin concentrations to return to base level. Each block contained two trials, lasting approximately 52 seconds.
During the task, each participant held a color disk and controlled its horizontal movements by pressing corresponding buttons on the computer to select a column. Once the disk ceased moving, it would drop vertically to the lowest available space of the board within 2 seconds in that selected column. Both participants took turns moving a disk, with each one holding four disks in total within one trail. Task performance was assessed by the error rate, which was the proportion of moves violating the role requirements specified in the context.
fNIRS data acquisitionThe functional near-infrared spectroscopy device (fNIRS; NirSmart II-200Pro; Danyang Huichuang Medical Equipment Co., Ltd, Jiangsu, China) simultaneously collected cerebral neural data from each dyad at wavelengths of 730 nm and 850 nm with a sampling rate of 11 Hz. The task-relative oxyhemoglobin (HbO) and deoxyhemoglobin (HbR) concentrations were converted using the modified Beer-Lambert Law (Pellicer & Bravo, 2011). As the concentration of HbO is a sensitive marker for regional cerebral blood flow in fNIRS studies, our study focused on it (Hoshi, 2003). We used 12 emitters and 11 detectors with 3 cm optode separation to form 31 channels.
The electromagnetic spatial position tracking system (FASTRAK; Polhemus, USA) was employed to determine the spatial positions of all emitters, detectors, and channels. The international 10-20 system, with NZ, CZ, AL, and AR serving as reference points, was utilized for localization. The spatial coordinates of the Montreal Neurological Institute (MNI) were estimated for each emitter, detector, and channel position by the NIRS_SPM toolbox on MATLAB (Xia et al., 2013) (Table S1). The optode panel primarily covered the PFC with the Fpz electrode as the reference point and covered the r-TPJ with the P6 electrode as the reference point. The specific cortex including dorsolateral prefrontal cortex (dlPFC), frontopolar cortex (FPC), inferior prefrontal gyrus (IFG), orbitofrontal cortex (OFC), supramarginal gyrus (SMG), angular gyrus (AG), superior temporal gyrus (STG), somatosensory association cortex (SAC) (Fig. 1d).
Assessing the performance of pattern gameThe task performance was evaluated by the error rate, which was calculated as the percentage of incorrect moves relative to total moves under each condition during the Pattern Game (Liu et al., 2017; Zhao et al., 2022). An incorrect move occurred when participants violated the goals and requirements of their assigned role. For example, the builder put disks in locations that did not match the target pattern; the helper obstructed the builder's construction of the target pattern; the hinderer helped the builder complete the reproduction of the target pattern. A lower error rate indicated that dyads or individuals performed better on the task.
fNIRS data analysisPreprocessingWe used the NirSpark package (Danyang Huichuang Medical Equipment Co., Ltd., China) to preprocess the fNIRS data. Motion artifacts for each channel were detected using a spline interpolation algorithm, which was commonly used for the advantage of correcting only pre-localized artifacts (Scholkmann et al., 2010). The data were bandpass filtered, ranging from 0.01 to 0.1 Hz, to remove physiological noise including respiration, cardiac activity, and low-frequency signal drift (Pan et al., 2024; Zhang et al., 2024).
Inter-brain SynchronizationWe conducted the wavelet transform coherence (WTC) analysis by the NirSpark package on the preprocessed data to assess IBS within dyads (Pan et al., 2024; Zhao et al., 2022; Zhao et al., 2024). To determine the frequency band of interest (FOI), task-state and resting-state IBS were averaged separately, followed by a series of paired sample t-tests to obtain the p-value (FDR-corrected). Significantly higher task-state IBS than the resting IBS was observed in two bands in the range of 0.015 - 0.022 Hz (period 45.45 - 66.67 s) and 0.026 - 0.039 Hz (period 25.47 - 38.16 s) (Fig. S1). The higher frequency band range was selected for two reasons. First, it reliably reflected the higher cognitive activities and excluded the interference of physiological data such as respiration and cardiac pulsation (Zhang et al., 2023). Second, each trial in the Pattern Game lasted approximately 26 s, which fits within the period range. Therefore, the choice of the frequency band range of 0.026-0.039 Hz as FOI was reasonable and effective. We averaged the IBS across the FOI. The IBS increment was calculated as the task-state IBS minus resting-state IBS, then averaged across four blocks within each condition. The IBS increment was subsequently computed and transformed into z-scores by applying Fisher z statistics.
Individual brain activityThe HbO for each block within the condition was superimposed and averaged. HbO time-series data were analysed using a general linear model (GLM) implemented in the NirSpark package. Regression coefficient β values were obtained by calculating the hemodynamic response function (HRF) from the real data and ideal design. β values reflected activation in the cerebral cortex of an individual. Higher β values represented higher levels of individual cortical activity.
Data statistical analysisWe performed the statistical analysis using SPSS 21.0 (IBM Corp., NY, USA). A mixed-design ANOVA was then conducted with GROUP (HUD vs. HC) as the between-subject variable and CONDITION (cooperation vs. competition) as the within-subject variable, followed by simple effects analysis for significant channels. Differences in neural and behavioral patterns between the HUD participants and the HC participants were determined using an independent samples t-test with FDR correction.
We calculated the Intraclass Correlation Coefficient (ICC) for clinical variables of the individuals with HUD (Liljequist et al., 2019). The results indicated that heroin craving (ICC = 0.19), addiction severity (ICC = 0.37), and protracted withdrawal symptoms (ICC = 0.36) were all predominantly influenced by individual-level variation, with no significant between-pair variation (ps > 0.077), suggesting no significant differences in individual clinical variables across different dyads. Additionally, with only two individuals per dyad, the non-independence of individuals nested within dyads is limited (Lee et al., 2018). Due to the random assignment of dyads, the inability to ignore within-dyad individual differences and the limited non-independence indicated by the ICC results, we assigned the dyad-level variable (IBS) to each individual within the dyad for subsequent individual-level analyses.
To reveal the relationships between behavioral performance, addiction-related indicators scale scores, and neural data, we conducted Pearson correlation analyses. Although the ICC results suggest that individual-level variance is dominant, providing a statistical basis for assigning IBS to individuals in exploratory correlation analyses, we further validated our core findings using a multilevel mediation model, which is the most appropriate method to account for the nested structure of our dyadic data in the final hypothesis testing (Preacher et al., 2010). We conducted the multilevel mediation analysis to confirm the mediating mechanism using a Bayesian approach implemented in the brms package in R (Bürkner, 2017). This approach retains individual differences and preserves both levels of analysis. The model included Craving as the independent variable, IBS as the mediator, and Error as the dependent variable, with a random intercept for dyads to control for within-dyad dependence. Statistical inference was based on 95% credible intervals obtained from the posterior distribution of the indirect effect.
We conducted a network analysis using JASP 0.19.3 to integrate variables influencing the performance of HUD participants under the cooperative conditions. Each node represented a core variable, including addiction-related symptoms of HUD participants, IBS, individual brain activity, and behavioral performance. In our study, the Pearson correlation coefficient was used to assess the edge weight between the nodes due to its computational robustness in small samples and a finite number of variables, avoiding the network becoming too sparse and the unstable centrality indicators (Epskamp & Fried, 2018). The threshold of |r| > 0.2 was set to exclude statistically defined weak correlations while balancing network sparsity with biological plausibility (Cohen, 1988). Thicker edges represented stronger associations. The centrality, including strength, closeness, and betweenness, was measured to identify the most influential variables within the network (Opsahl et al., 2010). The accuracy of the network connections was performed using 95% confidence intervals (CIs) for edge weights. These CIs were calculated through non-parametric bootstrapping with 1000 bootstrap samples. The stability of the network was assessed using a case-dropping bootstrap procedure with 1000 bootstrap samples.
ResultsDemographic informationThis study included 104 participants, comprising 54 HUD participants (32 males, age: M ± SD = 46.72 ± 8.79) and 52 HC participants (24 males, age: M ± SD = 44.15 ± 7.59). All participants were separately randomly paired in dyads, forming 27 HUD dyads and 26 HC dyads. Table 1 presents the demographic differences between the HUD and HC participants. The two groups showed no significant differences in gender (χ2(1) = 1.83, p = 0.177), age (t(104) = 1.61, p = 0.111, Cohen’s d = 0.31), and educational attainment (t(104) = -1.64, p = 0.104, Cohen’s d = -0.32). The assessment of heroin craving, protracted withdrawal, and addiction severity was described in the Method.
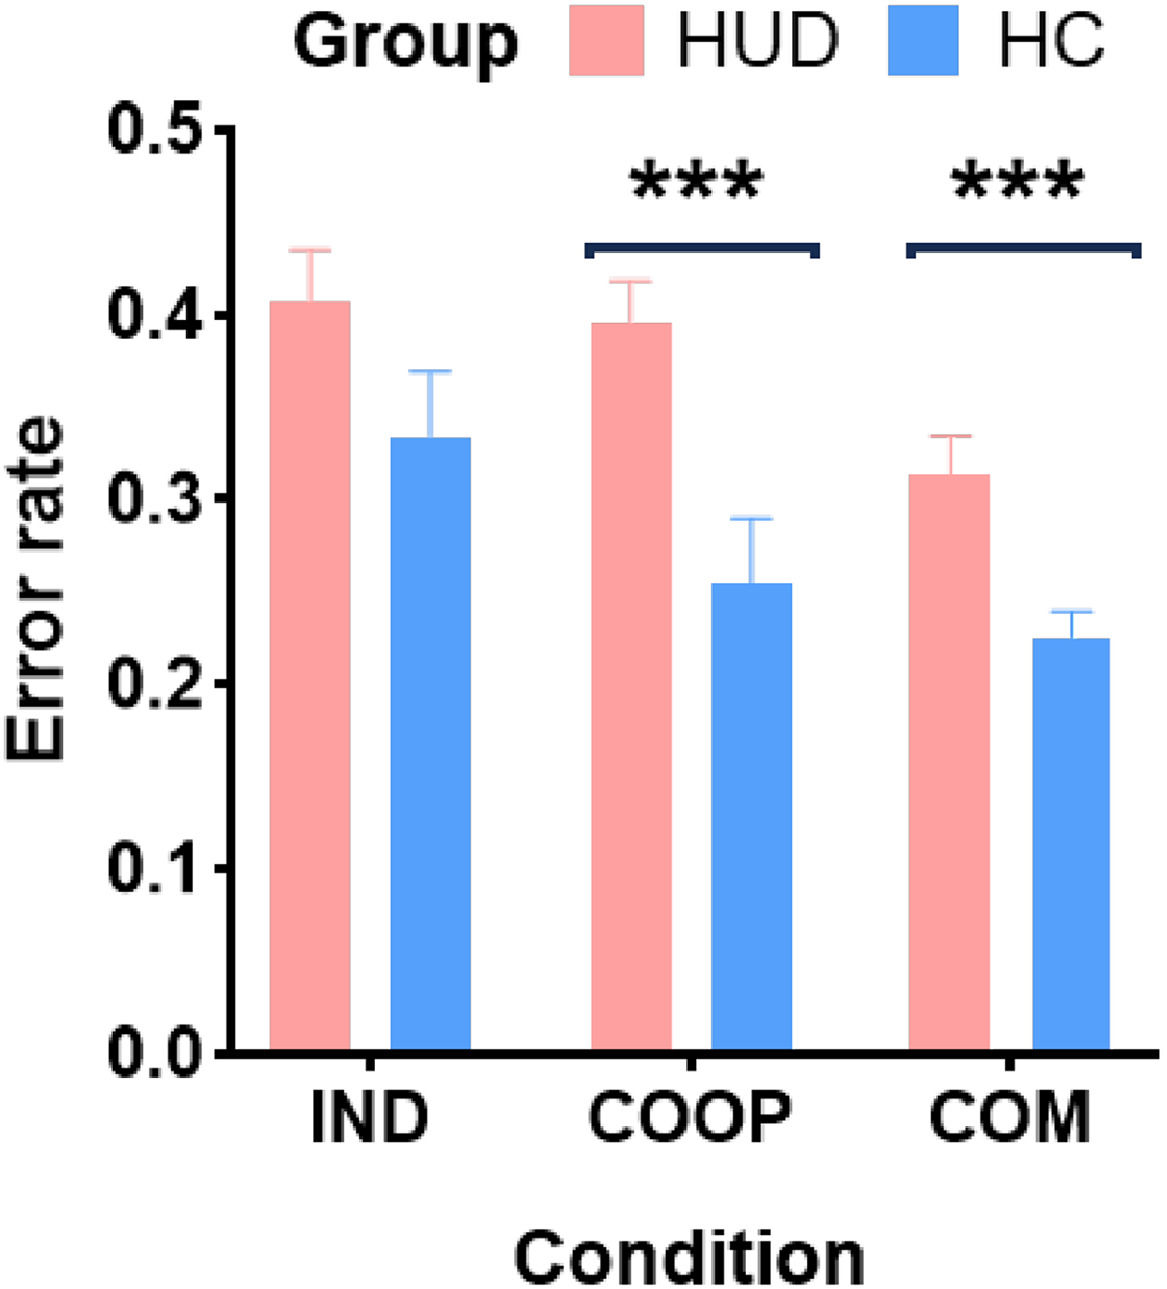
Behavioral performanceThe mean error rate in the Pattern Game task was used to evaluate the performance of the HUD and HC dyads in the turn-based interaction. To investigate the differences among different conditions, we further conducted a mixed-design ANOVA on error rate, with GROUP (HUD vs. HC) as a between-subject variable and CONDITION (independence vs. cooperation vs. competition) as a within-subject variable (Fig. 2). We found a significant interaction effect of CONDITION × GROUP (F(2, 50) = 3.48, p = 0.039, η2p = 0.12). Subsequent simple effect analysis demonstrated that the error rate between the HUD and HC dyads did not differ significantly under the independent condition, indicating that the ability to perform tasks alone did not affect interpersonal interaction performance. Therefore, the independent condition was not included in the analysis of subsequent neural results. Under both the cooperative and competitive conditions, the HUD dyads exhibited higher error rate compared to the HC dyads (p < 0.001), indicating the behavioral deficit both in the two interactions. Furthermore, the HUD dyads exhibited significantly lower error rate under the competitive condition than under both the independent (p = 0.002) and cooperative (p = 0.006) conditions, suggesting the competition predilection in HUD. The HC dyads exhibited significantly lower error rate both under the cooperative (p < 0.001) and competitive (p < 0.001) conditions than the independent condition. Detailed information is presented in Table S2.

Task performance across the three conditions. Only significant group differences between HUD and HC dyads in the simple effect analysis are annotated on the plot. Error lines are standard errors. HUD: dyads with heroin use disorder, HC: healthy control dyads, IND: independent condition, COOP: cooperative condition, COM: competitive condition. *p < 0.05, **p < 0.01, ***p < 0.001.
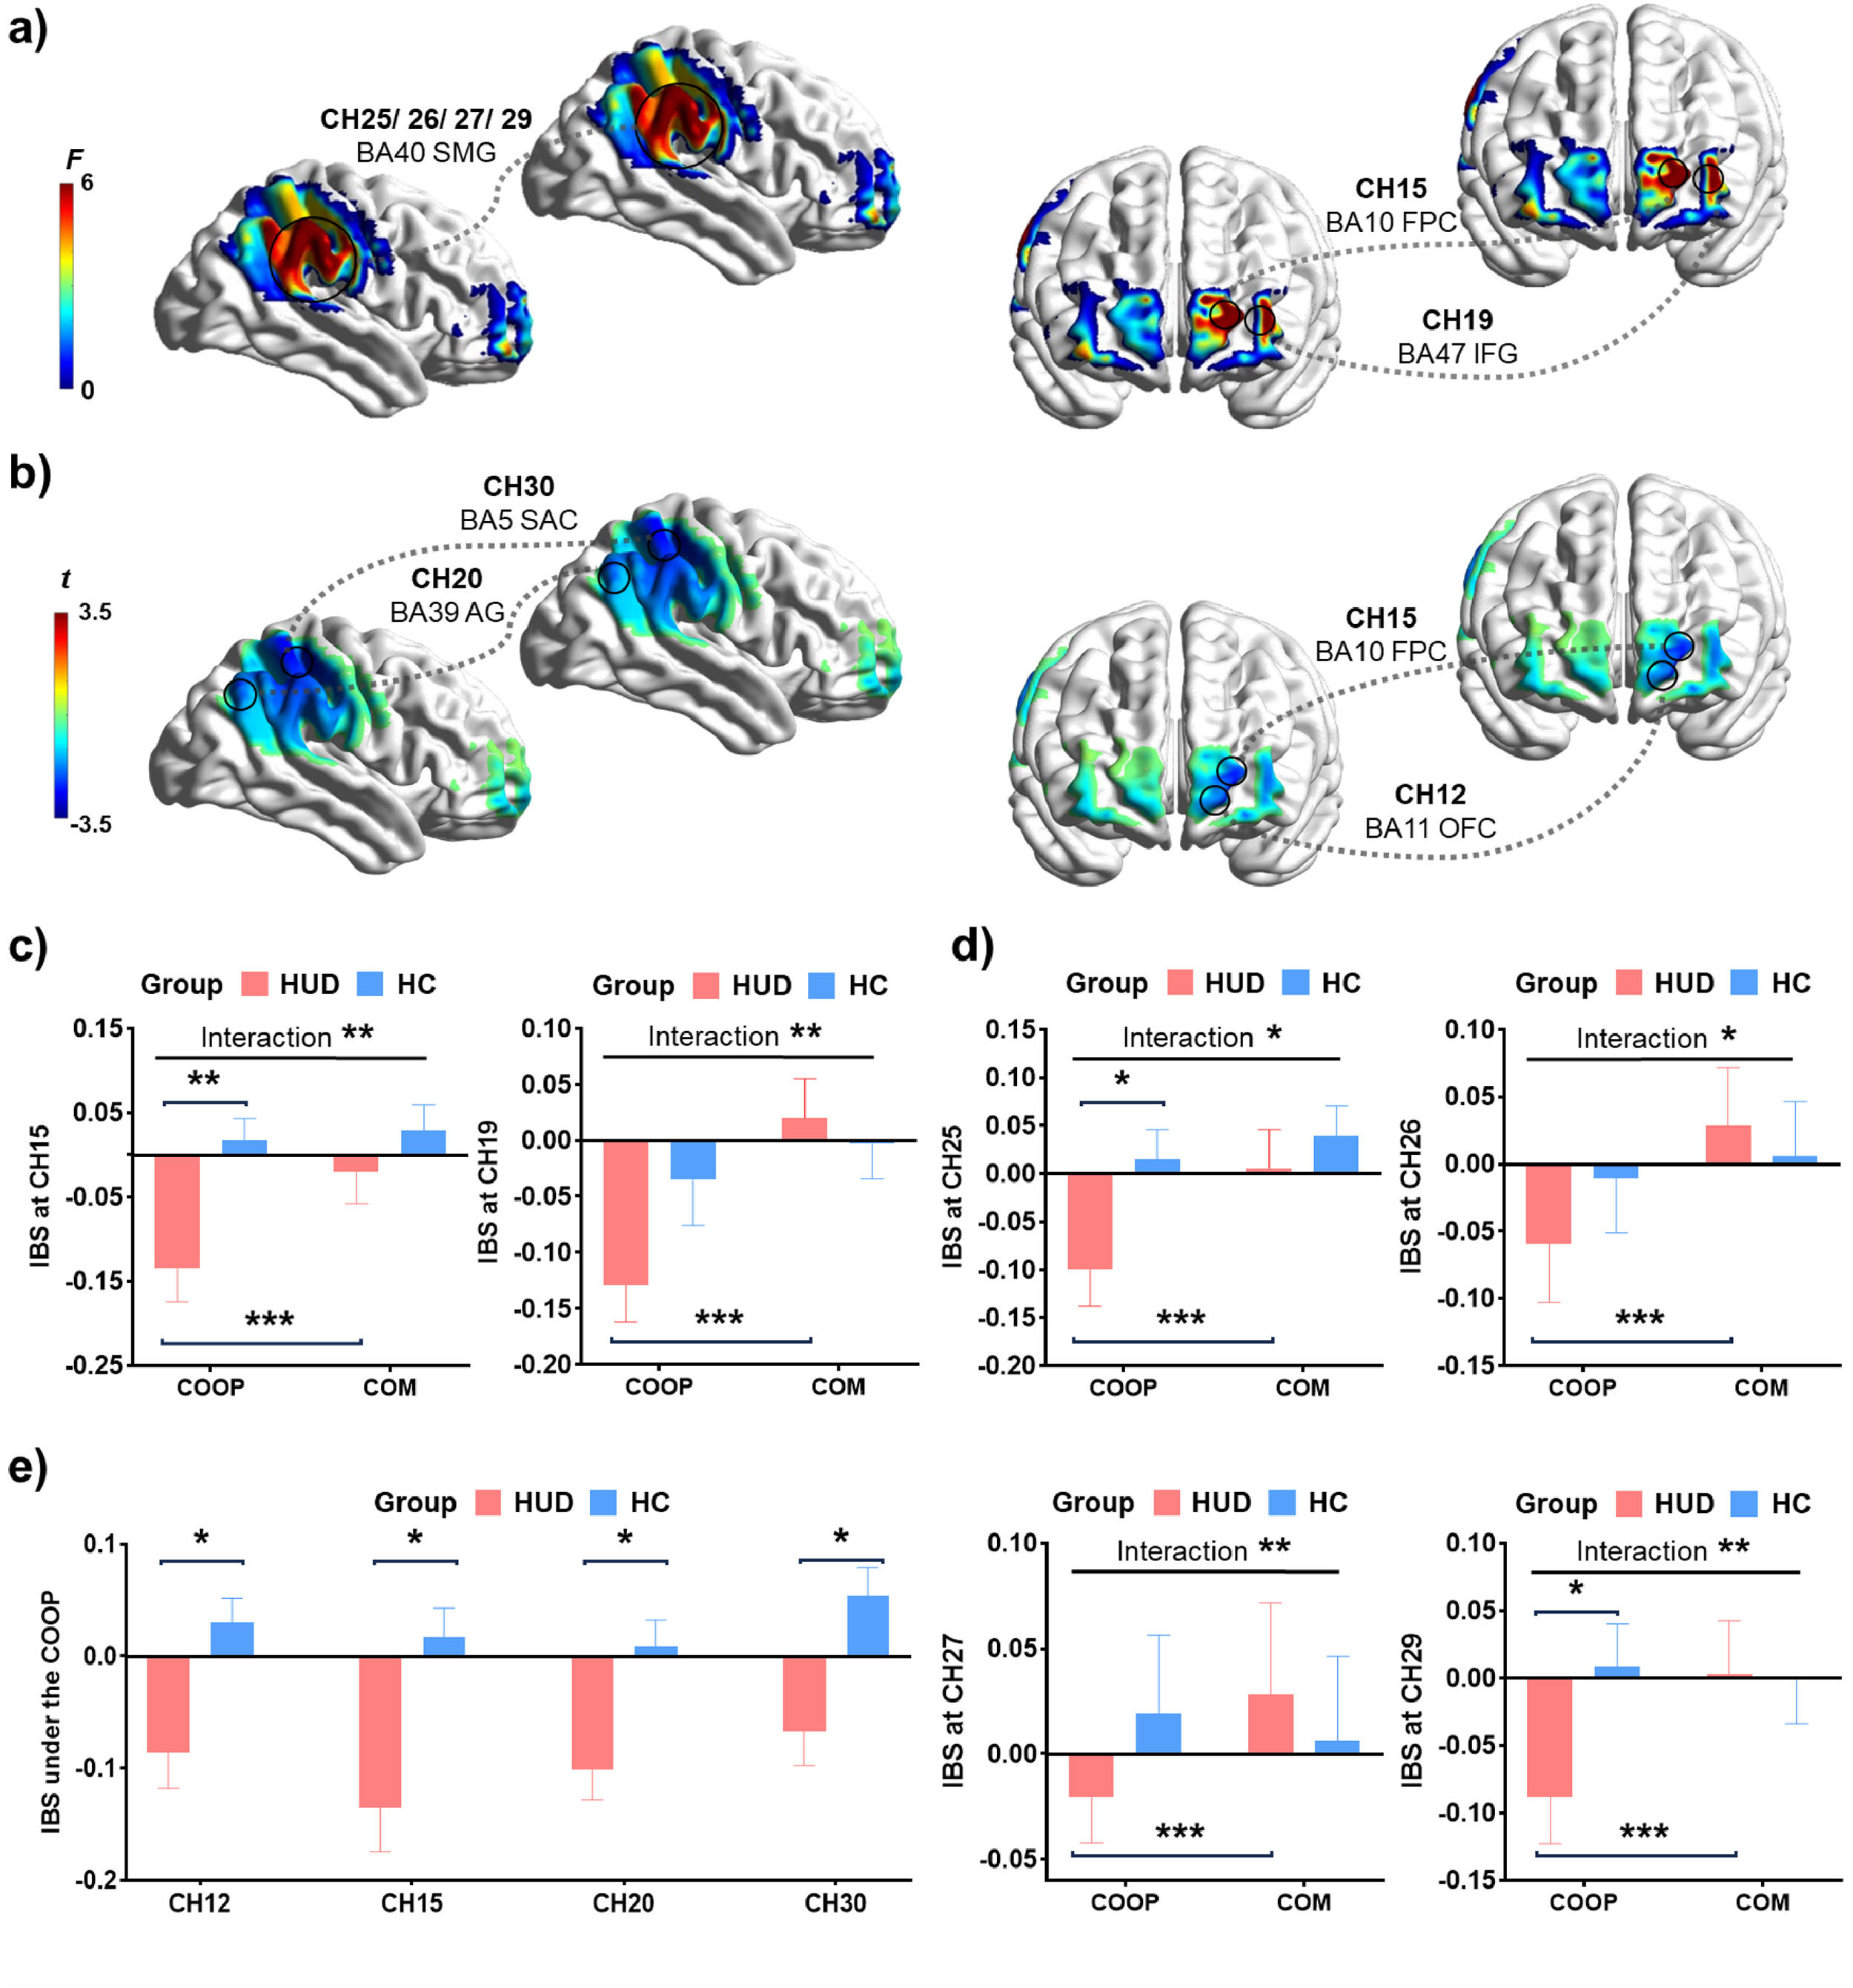
To investigate the differences between cooperation and competition in HUD, we conducted a mixed-design ANOVA on the IBS increment, with GROUP (HUD vs. HC) as a between-subject variable and CONDITION (cooperation vs. competition) as a within-subject variable. We observed a significant interaction effect of CONDITION × GROUP in the PFC at CH15 (F(1, 51)= 14.61, pFDR = 0.007, η2p = 0.22; frontopolar cortex, FPC), at CH19 (F(1, 51) = 12.33, pFDR = 0.001, η2p= 0.20; inferior prefrontal gyrus, IFG), and the supramarginal gyrus (SMG) in the r-TPJ at CH25 (F(1, 51) = 9.52, pFDR = 0.020, η2p = 0.16), CH26 (F(1, 51) = 7.08, pFDR = 0.054, η2p = 0.12), CH27 (F(1, 51) = 14.18, pFDR = 0.007, η2p = 0.22), and CH29 (F(1, 51) = 9.93, pFDR = 0.007, η2p = 0.16) (Fig. 3a). The simple effect analysis demonstrated that the IBS increment at these channels in the HUD dyads under the competitive condition was significantly higher than that under cooperative conditions (all ps < 0.001) (Fig. 3c, d). However, there was no significant difference in the IBS increment among HC participants between the cooperative and the competitive conditions. Under the cooperative condition, the HUD dyads exhibited lower IBS increment at CH15 (p = 0.002), CH25 (p = 0.024) and CH29 (p = 0.047) compared to the HC dyads, while no significant difference under the competition condition between the two groups.

Inter-brain synchronization. a)F-map of IBS increment on interaction effects of GROUP and CONDITION. b)t-map of IBS increment in the r-TPJ and PFC under the cooperative condition between HUD dyads and HC dyads. c) IBS increment in the PFC for the HUD dyads and HC dyads under the cooperative and competitive conditions. d) IBS increment in the r-TPJ for the HUD dyads and HC dyads under the cooperative and competitive conditions. e) IBS increment differences between the HUD dyads and HC dyads under the cooperative condition. Error lines are standard errors. HUD: dyads with heroin use disorder, HC: healthy control dyads, IND: independent condition, COOP: cooperative condition, COM: competitive condition. *p < 0.05, **p < 0.01, ***p < 0.001.
To further identify cooperation-related deficits in HUD, we performed a series of independent samples t-tests on IBS of each channel between the HUD and the HC dyads under the cooperative condition. This analysis indicated significantly lower IBS increments under the cooperative condition in HUD relative to HC dyads at multiple channels including CH12 (t(51) = -3.04, pFDR = 0.031, Cohen’s d = -0.84; orbitofrontal cortex, OFC), CH15 (t(51) = -3.21, pFDR = 0.031, Cohen’s d = -0.89; FPC), CH20 (t(51) = -3.04, pFDR = 0.031, Cohen’s d = -0.84; angular gyrus, AG), and CH30 (t(51) = -3.09, pFDR = 0.031, Cohen’s d = -0.85; somatosensory association cortex, SAC) (Fig. 3b, e, Table S3).
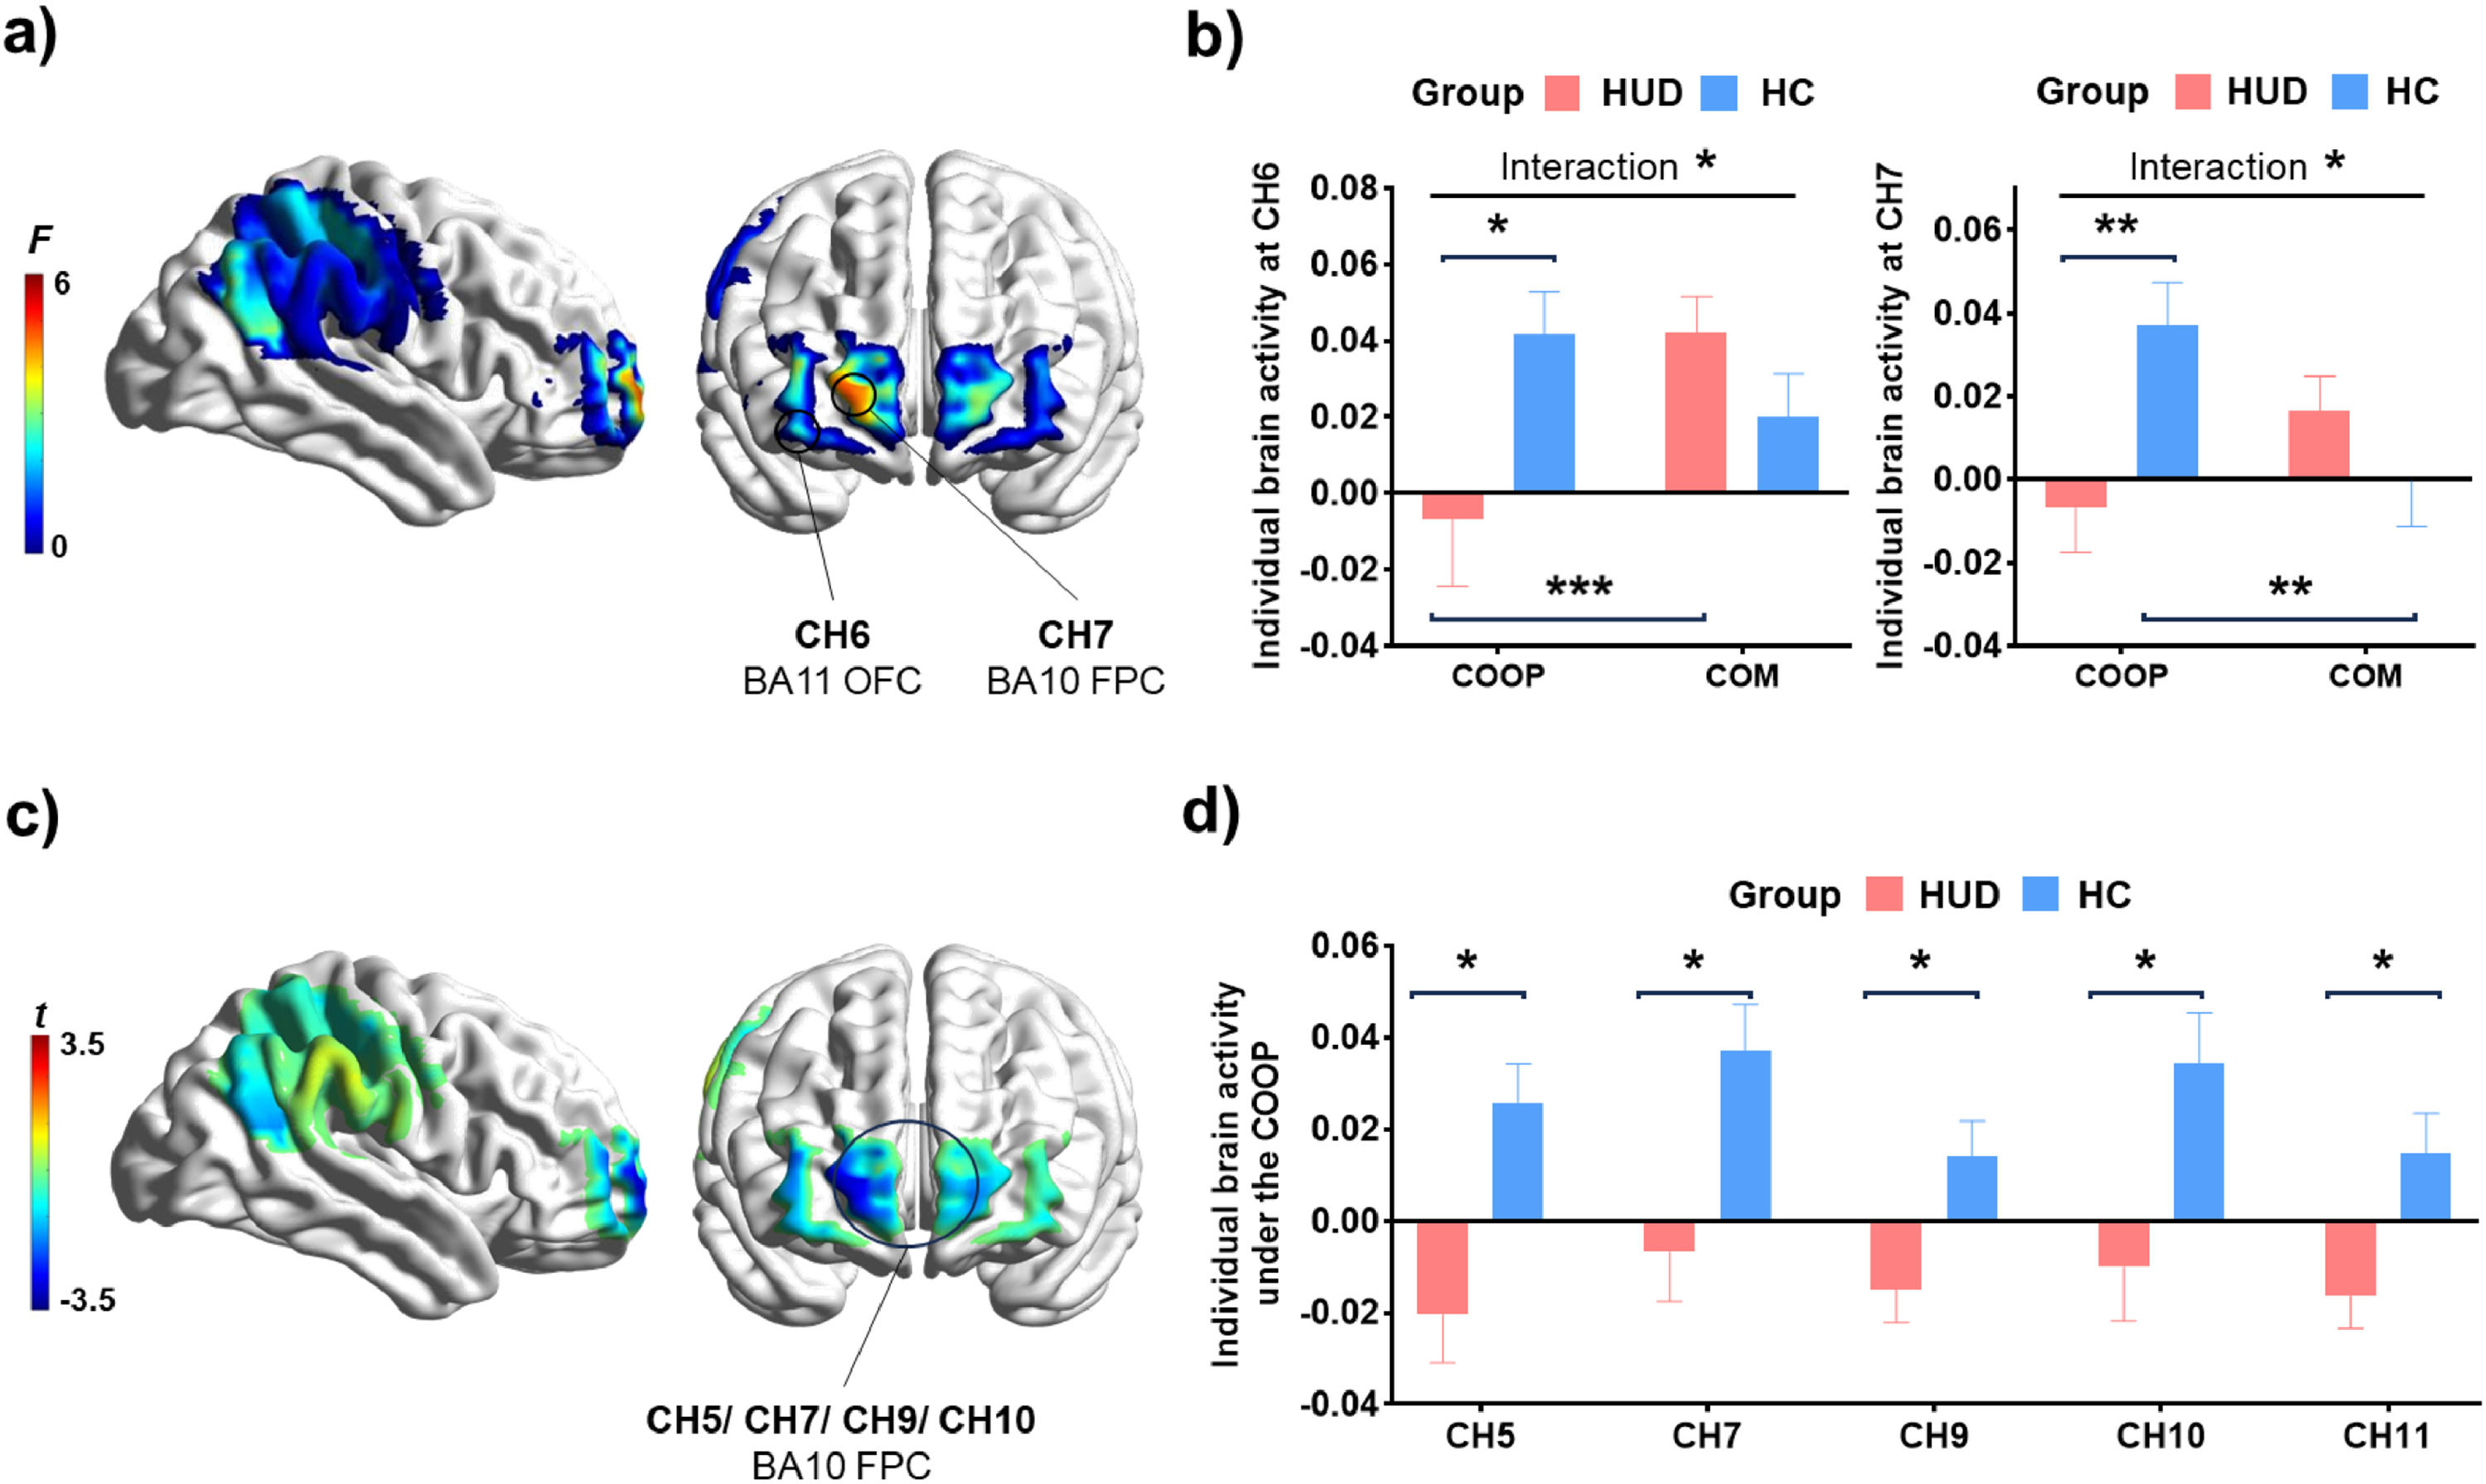
Individual brain activityThe mixed-design ANOVA on individual brain activity (β values) was conducted, with GROUP (HUD vs. HC) as a between-subject variable and CONDITION (cooperation vs. competition) as a within-subject variable. The results revealed a significant interaction effect of GROUP × CONDITION in the PFC at CH6 (F(1, 104) = 11.19, pFDR = 0.028, η2p = 0.10; OFC) and CH7 (F(1, 104) = 10.29, pFDR = 0.028, η2p= 0.09; FPC) (Fig. 4a). Simple effects analysis further indicated that HUD participants exhibited significantly lower β values at CH6 under the cooperative condition compared to the competitive condition (p = 0.001), whereas the HC participants exhibited significantly higher β values at CH7 under the cooperative condition than under the competitive condition (p = 0.007) (Fig. 4b). Under the cooperative condition, the HUD participants exhibited lower β values at CH6 (p = 0.023) and CH7 (p = 0.001) compared to the HC participants. The two groups showed no significant differences under the competition condition.

Individual brain activity. a)F-map of the interaction effects of GROUP and CONDITION on individual brain activity. b) Individual brain activity of the groups and conditions at CH6 and CH7 in the PFC. c)t-map of individual brain activity under the cooperative condition between the HUD and the HC participants. d) Differences in individual brain activity between HUD participants and HC participants under the cooperative condition. Error lines are standard errors. HUD: participants with heroin use disorder, HC: healthy control participants, COOP: cooperative condition, COM: competitive condition.*p < 0.05, **p < 0.01, ***p < 0.001.
To further identify cooperation-related deficits in HUD, we performed a series of independent samples t-tests on β values of each channel between the HUD and the HC dyads under the cooperative condition. This analysis indicated significantly lower β values under the cooperative condition in HUD relative to HC dyads in the FPC at multiple channels, including CH5 (t(104) = -3.42, pFDR = 0.031, Cohen’s d = -0.67), at CH7 (t(104) = -2.93, pFDR = 0.050, Cohen’s d = -0.57), CH9 (t(104) = -2.68, pFDR = 0.050, Cohen’s d = -0.52), CH10 (t(104) = -2.78, pFDR = 0.050, Cohen’s d = -0.54), and CH11 (t(104) = -2.74, pFDR = 0.050, Cohen’s d = -0.53) (Fig. 4c, d, Table S4).
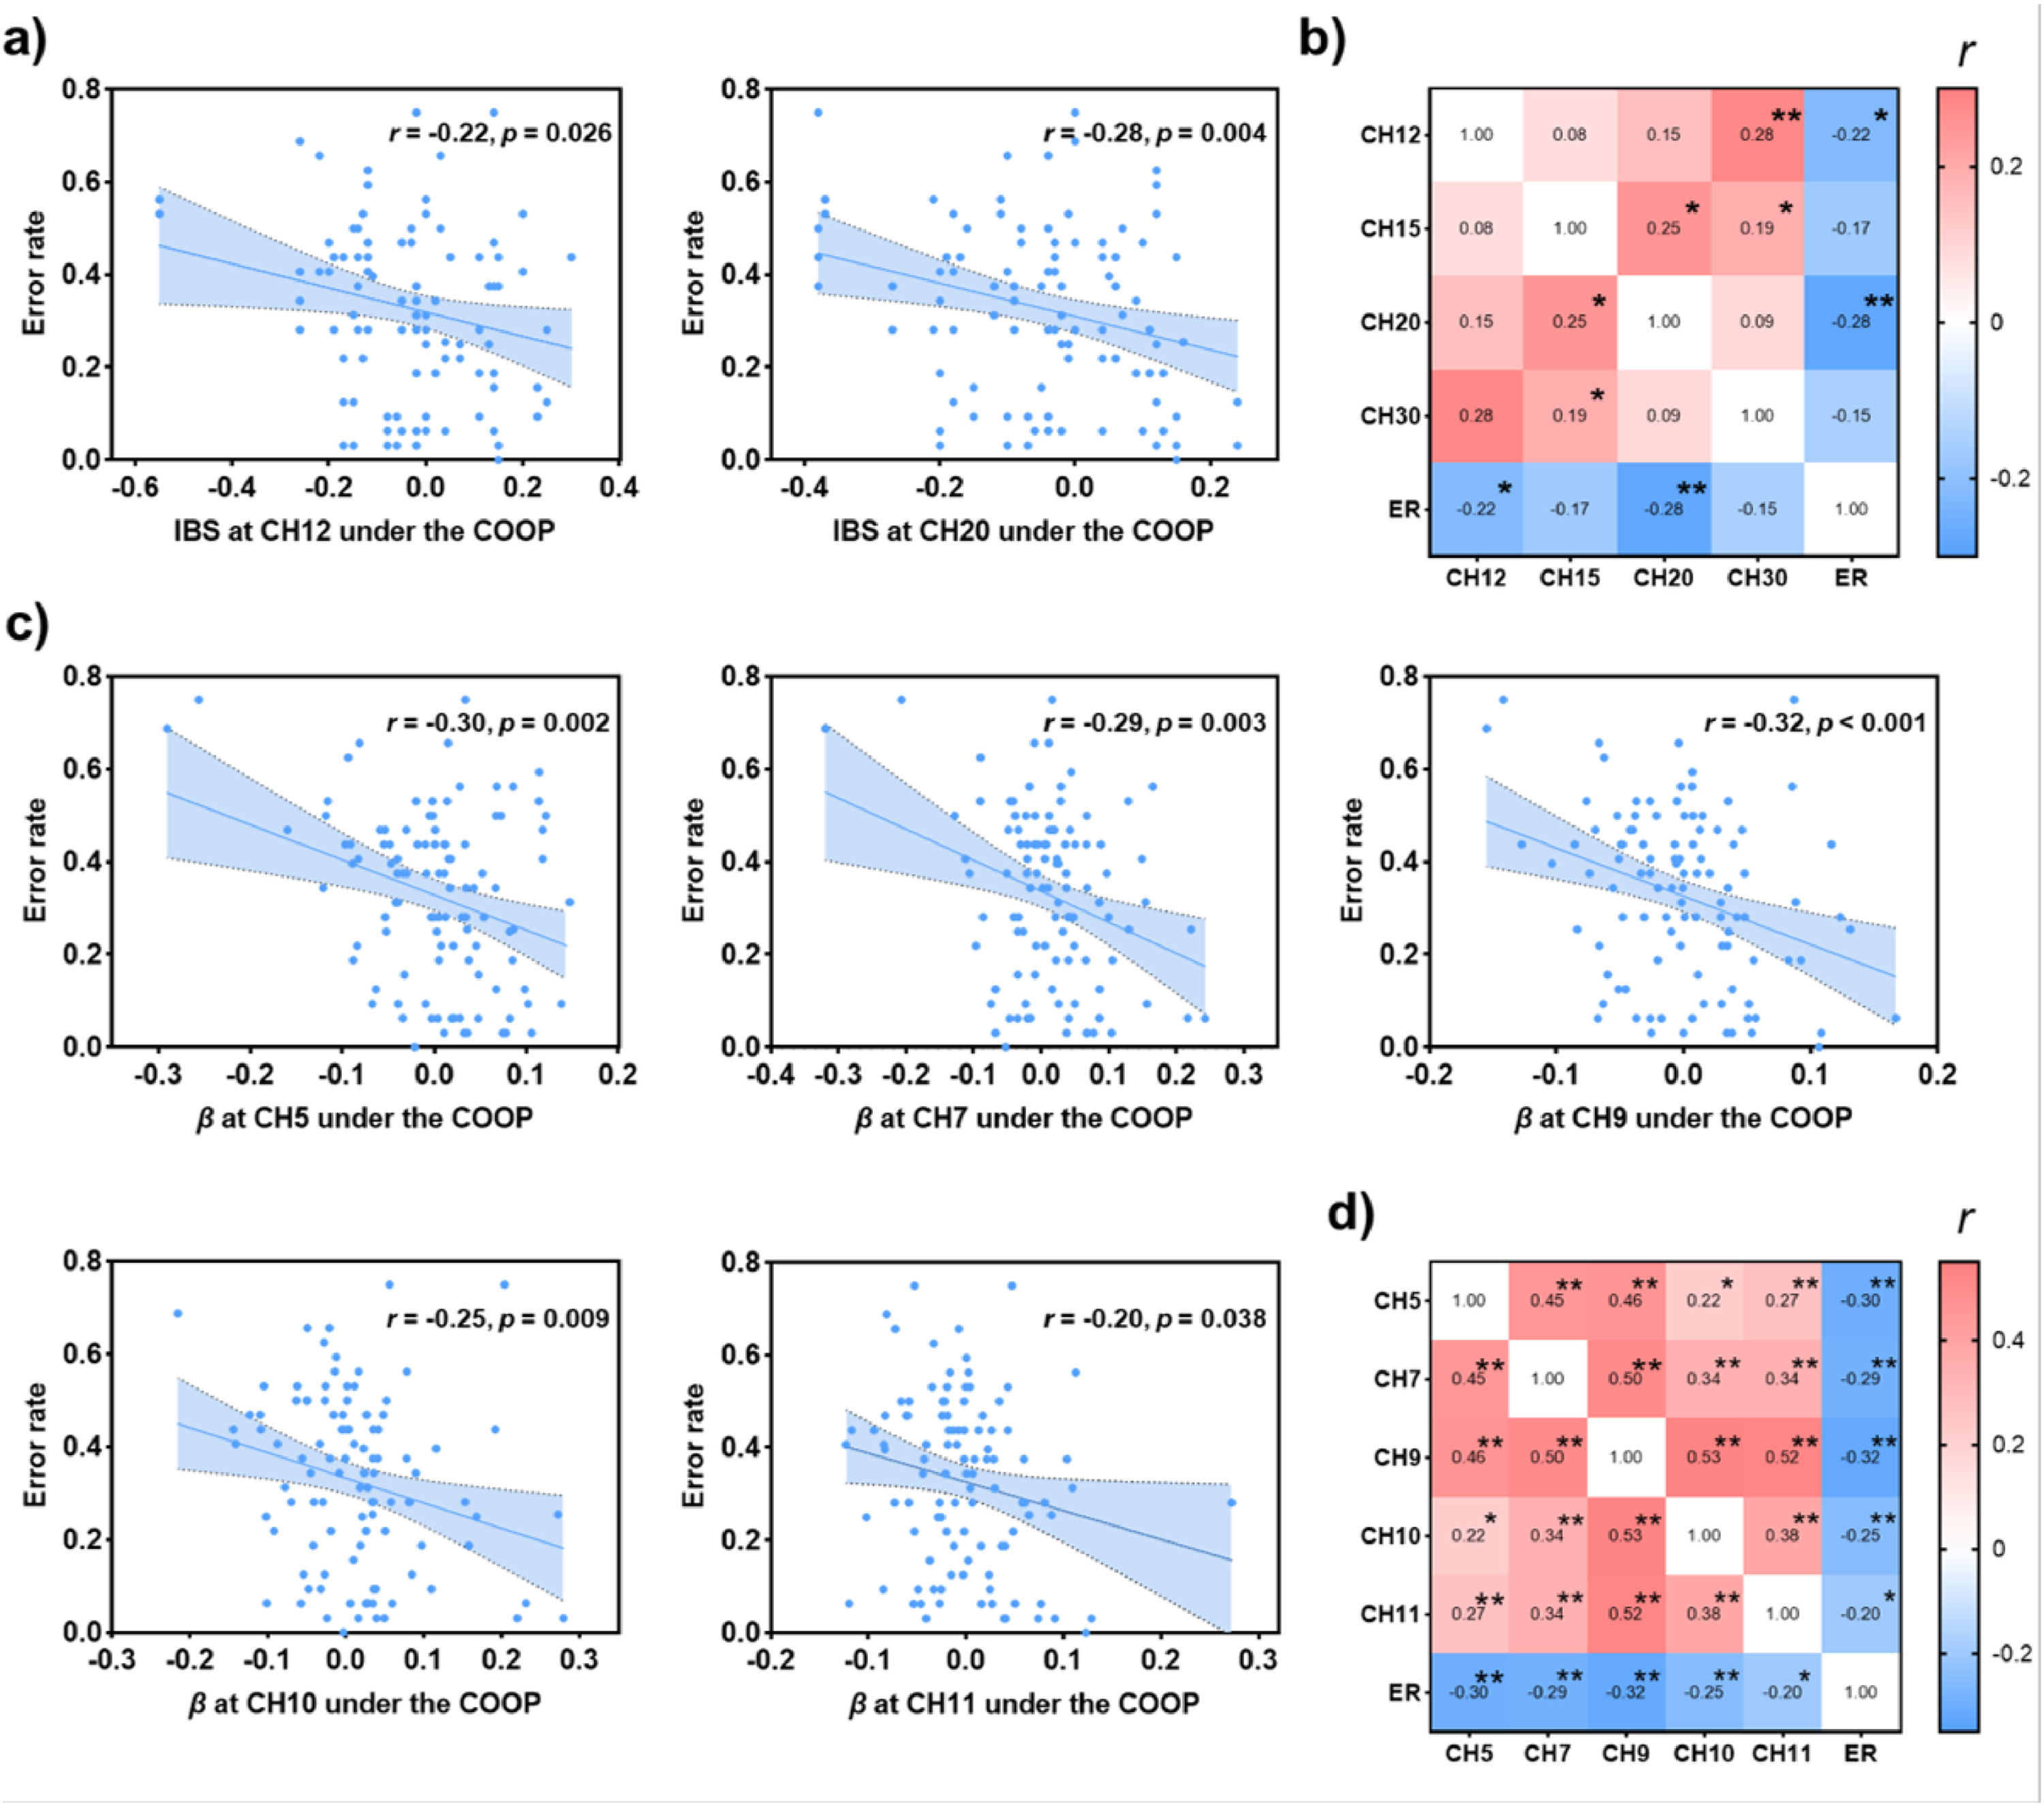
CorrelationPearson’s correlation analysis revealed the correlation between neural responses and behavioral performance. There was a significant negative correlation between the IBS increment (in the PFC and r-TPJ) and error rate under the cooperative condition (CH12: r = -0.216, p = 0.026; CH20: r = -0.277, p = 0.004) (Fig. 5a-b). The β values in the FPC were also significantly negatively correlated with the error rate under the cooperative condition (CH5: r = -0.303, p = 0.002; CH7: r = -0.290, p = 0.003; CH9: r = -0.322, p < 0.001; CH10: r = -0.251, p = 0.009; CH11: r = -0.202, p = 0.038) (Fig. 5c-d).

The correlation between neural response and behavioral performance under the cooperative condition. a) The significant correlations between IBS increment and error rate. b) The correlation matrix map of IBS and error rate. c) The significant correlations between β values and error rate. d) The correlation matrix map of β values and error rate. In each scatter plot, the dots represent all data samples, the solid line indicates the least-squares fit, and the shaded area between the dotted lines represents the 95% confidence interval of the regression line. In each matrix map, the color bar denotes the degree of the Pearson correlation coefficient. COOP: cooperative condition, ER: error rate under the cooperative condition. *p < 0.05, **p < 0.01, ***p < 0.001.
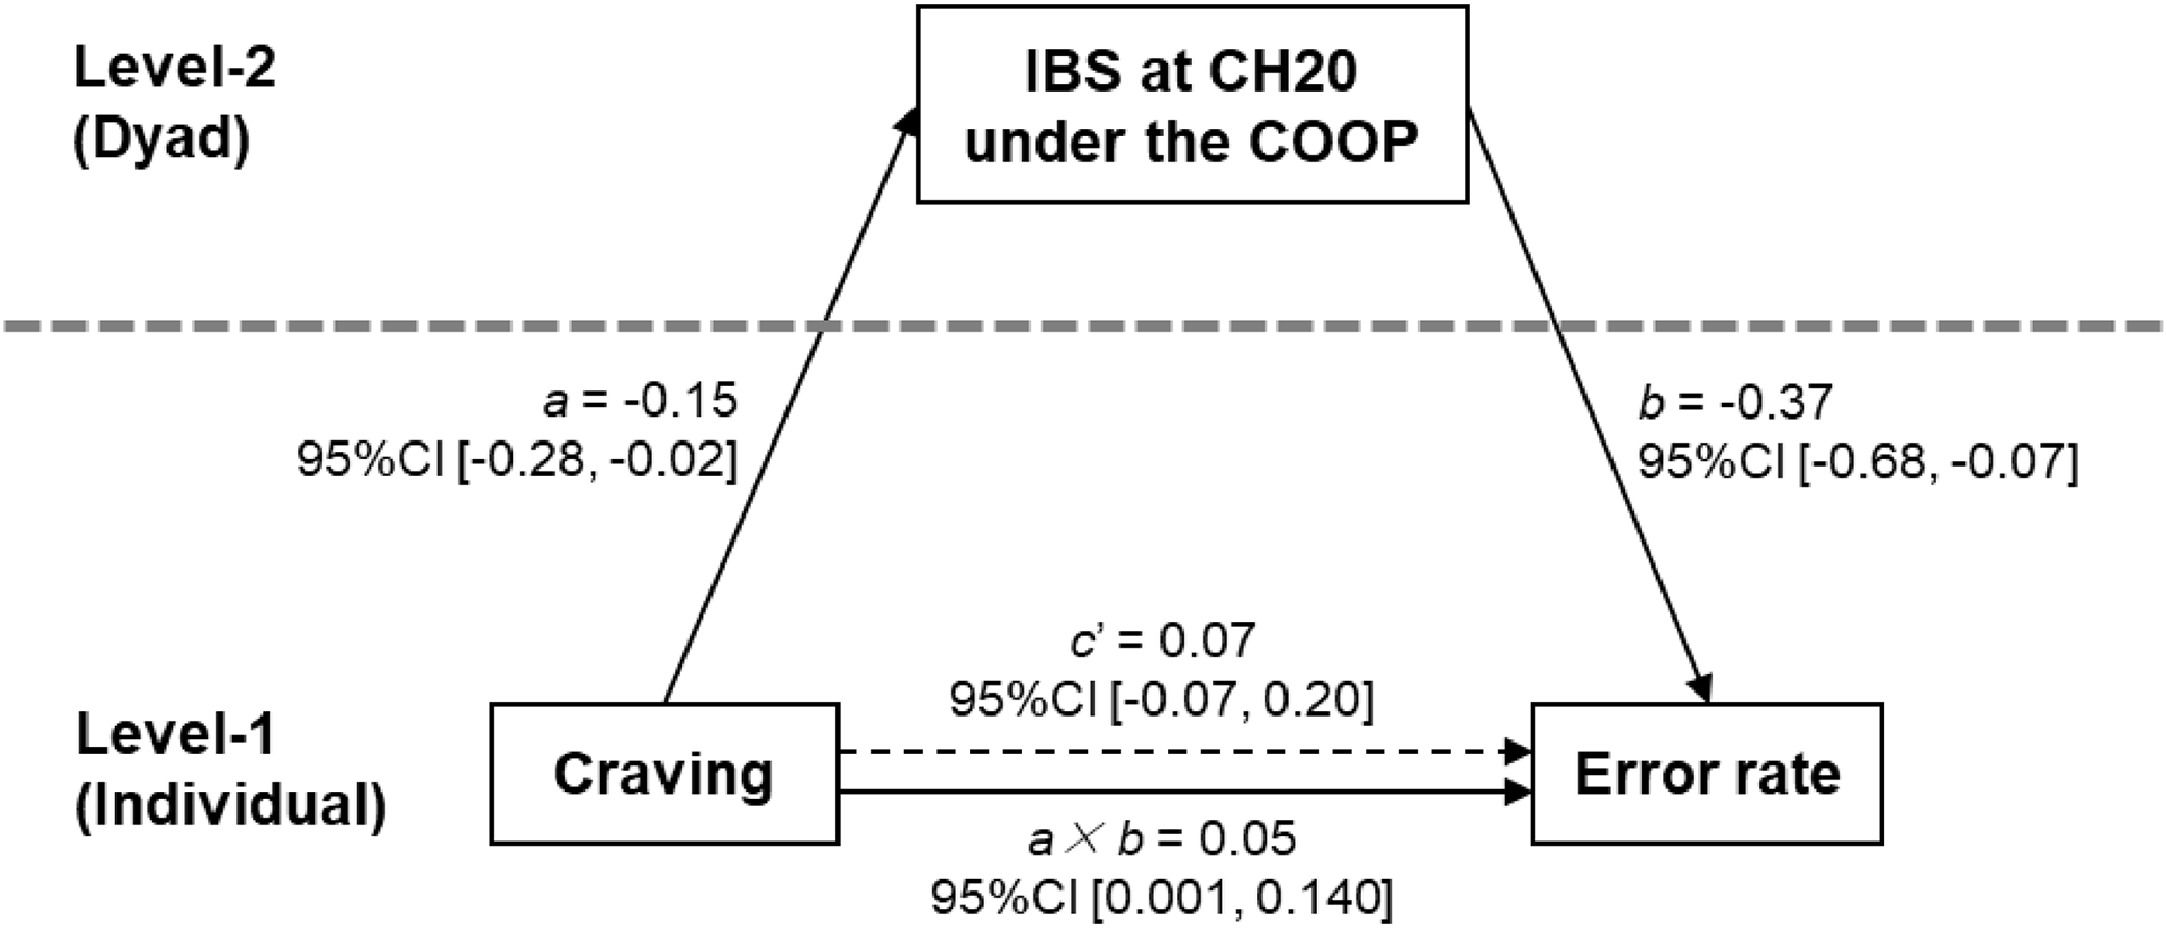
HUD participants exhibited a significant correlation between heroin craving, IBS increment, and error rate under the cooperative condition (Fig. S2). To further elucidate the relationship among these variables while accounting for the nested structure of the data, we employed a multilevel mediation model. The results confirm that craving had a significant negative effect on IBS increment at CH20 under the cooperative condition (α = -0.15, 95% CI = [-0.28, -0.02]), and the IBS increment at CH20 exhibited a significant negative effect on error rate under the cooperative condition (b = -0.37, 95% CI = [-0.68, -0.07]). Furthermore, we observed a significant total indirect effect (a × b = 0.05, 95% CI = [0.001, 0.140]) of heroin craving on the error rate via the IBS at CH20 under the cooperative condition, indicating that the IBS at CH20 mediated the effect of heroin craving on the error rate under the cooperative condition (Fig. 6). Notably, after controlling for IBS increment at CH20, the direct effect of heroin craving on error rate under the cooperative condition was no longer significant (c' = 0.07, 95% CI = [-0.07, 0.20]). Furthermore, after controlling for years of heroin use and abstinence duration, the model results remained largely consistent with the main model, with the lower bound of the indirect effect's confidence interval slightly below zero, which can be considered marginally significant (a = -0.14, 95% CI [-0.28, -0.01]; b = -0.37, 95% CI [-0.67, -0.07];a × b = 0.049, 95% CI [-0.000, 0.136]; c' = 0.06, 95% CI [-0.08, 0.20]).

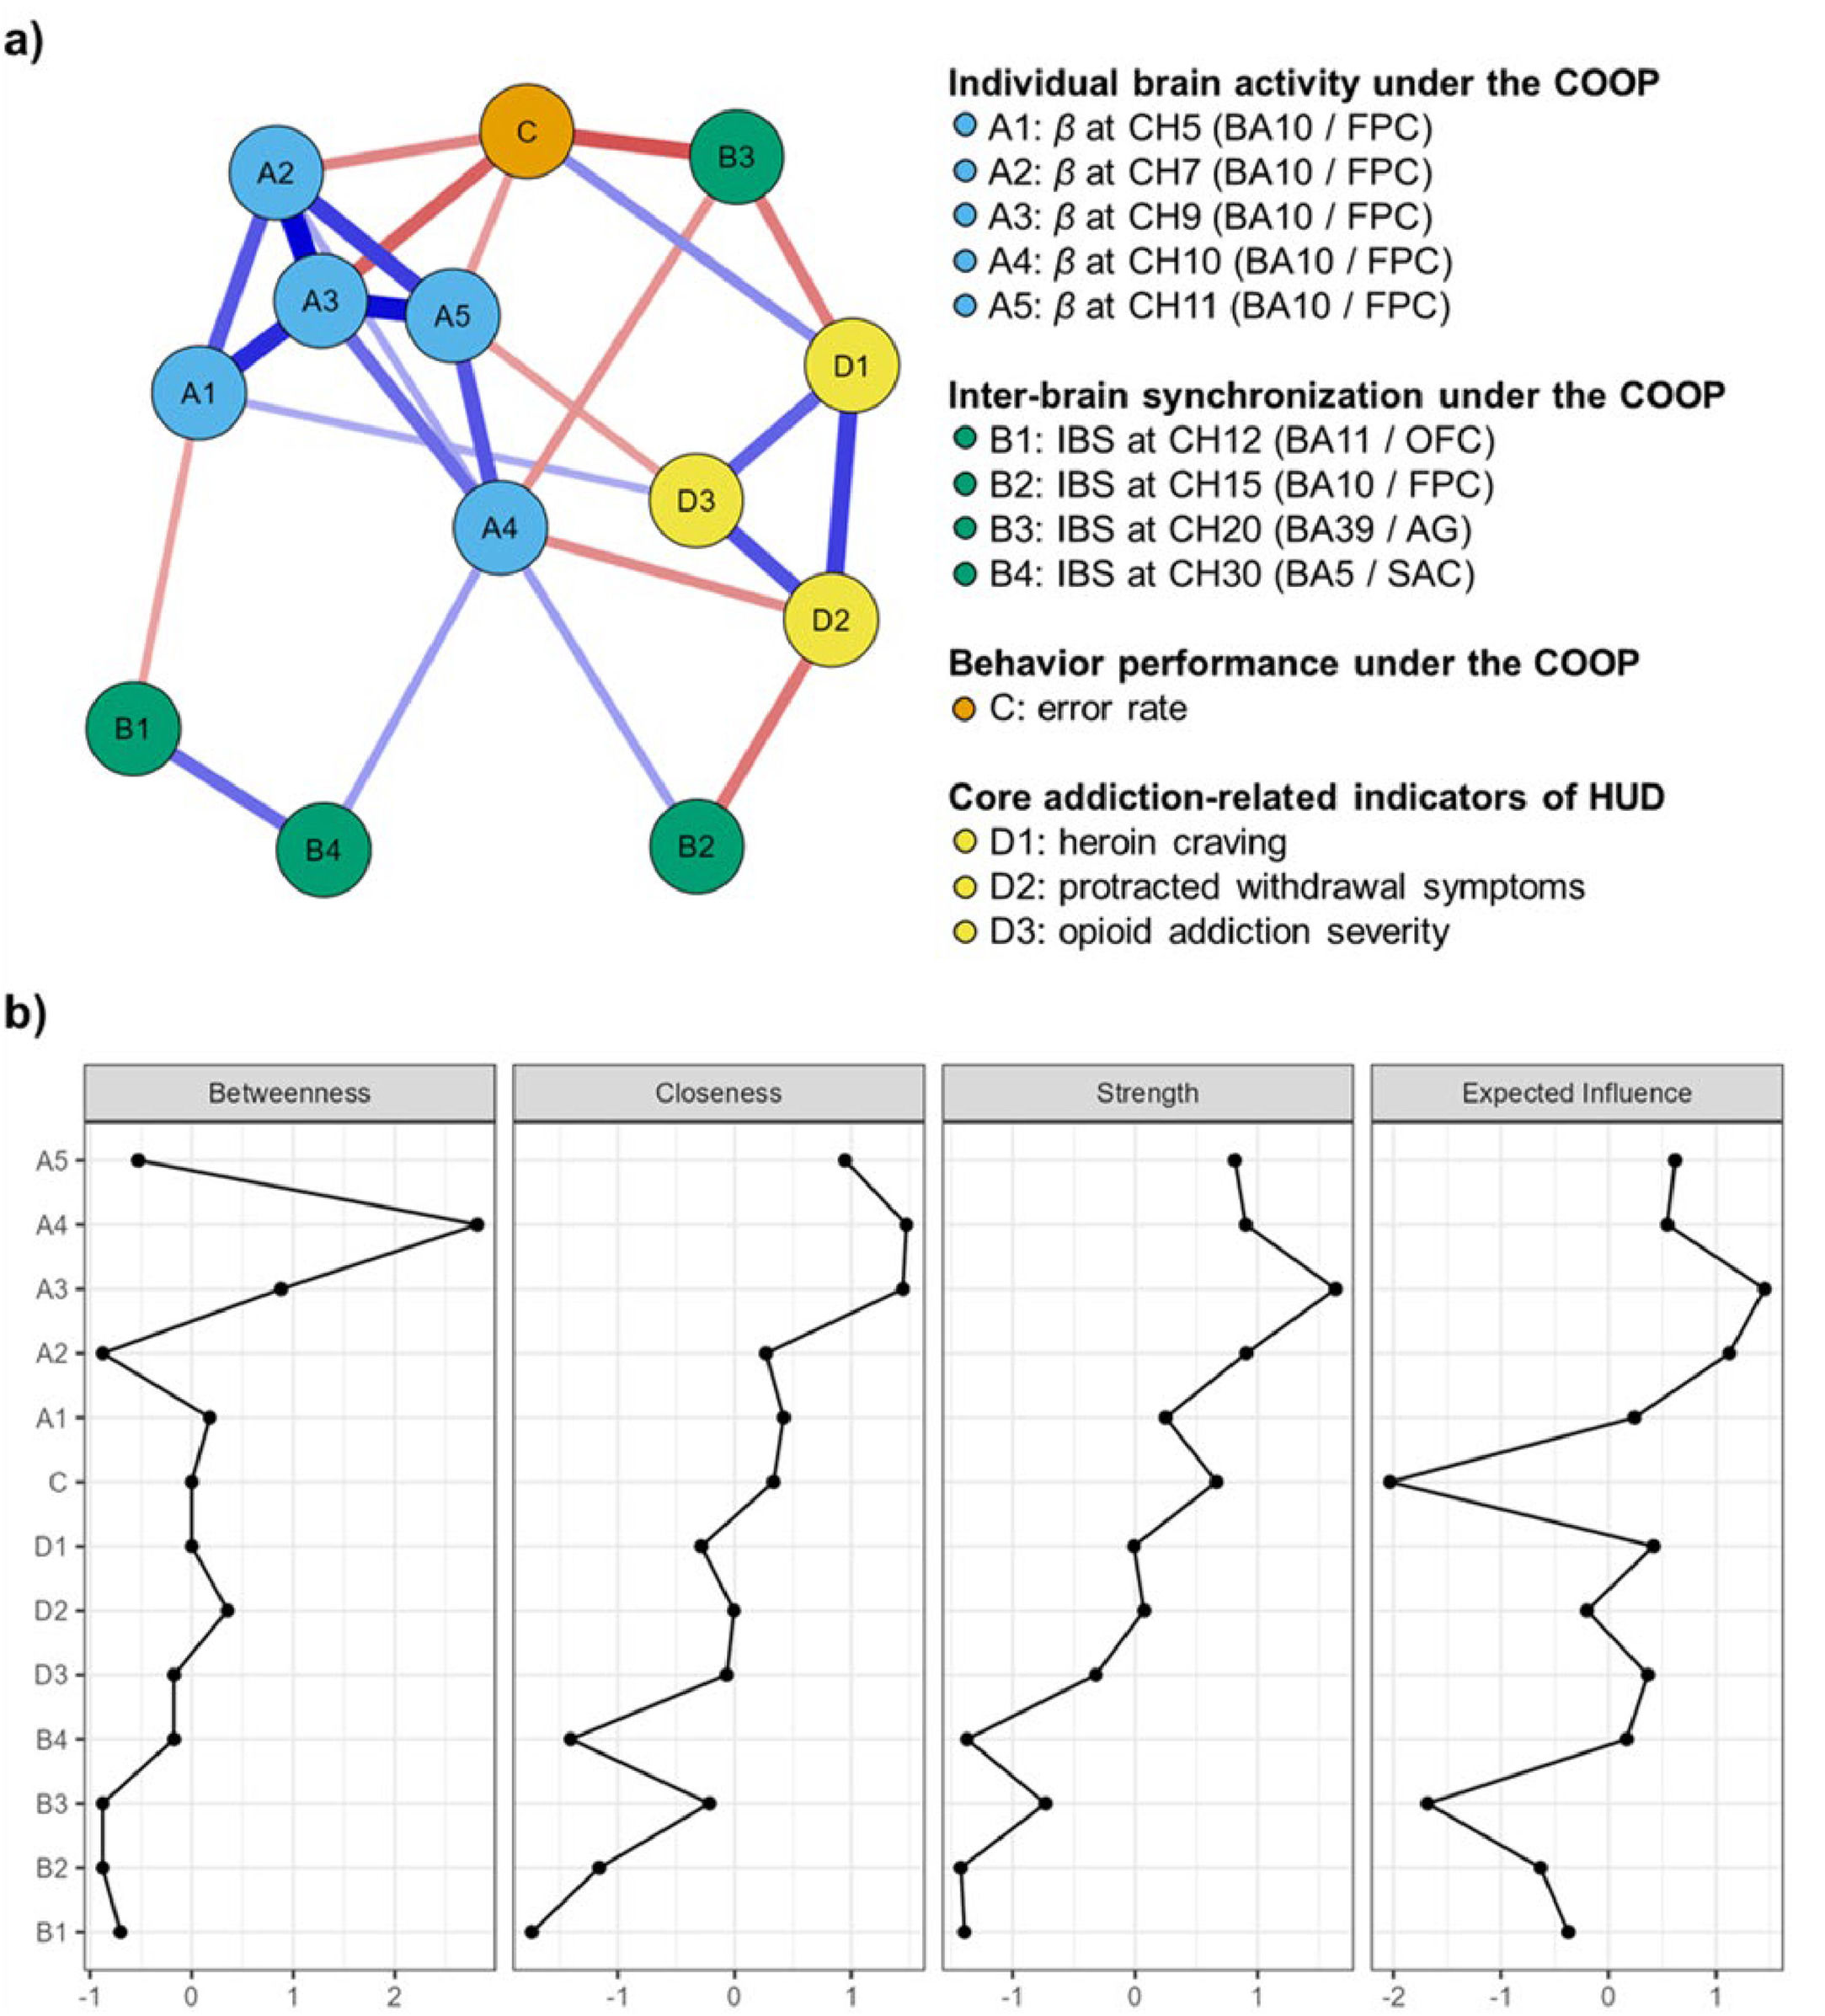
A network analysis was conducted to identify the most critical indicators and to deepen understanding of the relationships between neural signatures, behavioural performance, and addiction-related symptoms in individuals with HUD under the cooperative condition (Fig. 7a). In the network, nodes represent those variables mentioned above. Among those nodes, IBS in the AG at CH20 exhibited a stronger correlation with error rate under the cooperative condition (Table S5). The accuracy of edge weights was estimated using bootstrap-derived 95% non-parametric confidence intervals (CIs). The 95% CIs for the edge weights were relatively wide, suggesting substantial overlap between some edges; thus, edge rankings should be interpreted with caution (Fig. S3a). Finally, the stability of the centrality indices, including betweenness, closeness, and node strength, was assessed using a case-dropping bootstrap approach (Fig. 7b). The centrality stability coefficients were greater than 0.25, confirming that the network was stable (Fig. S3b). Since strength centrality was estimated with higher reliability, it was selected as the primary metric for identifying the most relevant variables. The three nodes with the highest strength centrality were β values in the FPC at CH9, CH7, and CH10, respectively (Table S6).

Symptom–brain network in individuals with HUD. a) The network structure of neural signatures, behavioral performance under the cooperative condition, and addiction-related indicators of HUD participants. The blue lines denote positive correlations, and red lines denote negative ones. The thickness and brightness of each edge reflect the correlation strength between the nodes. b) Centrality plots for the correlation in the network of each node. HUD: participants with heroin use disorder, COOP: cooperative condition.
The study explores the inter-brain and intra-brain neural mechanisms underlying the atypical cooperative and competitive interaction patterns during a real-time social interaction in HUD. As hypothesized, the HUD dyads exhibited a higher error rate and lower IBS in the PFC and r-TPJ, and decreased FPC activity under the cooperative condition. Compared with the cooperative condition, HUD participants showed a significant increase in IBS in the PFC and r-TPJ under the competitive condition, while the β values of the PFC also increased significantly. Critically, IBS in the r-TPJ mediated the effect of heroin craving on the error rate under the cooperative condition. These findings demonstrate impaired cooperative abilities and heightened competitive tendencies in HUD. The aberrant neural signatures during cooperation and competition among individuals with HUD are identified, providing reliable neurobiological biomarkers and neuromodulation targets for social dysfunction in drug addiction and other psychiatric disorders.
A diminished ability to cooperate compared to the healthy controlsIndividuals with HUD demonstrated both impaired cooperative ability and reduced motivation to engage in cooperation. Regarding behavioral performance, HUD dyads exhibited a higher error rate under the cooperative condition than under the competitive condition. This pattern was largely consistent with previous studies showing that chronic heroin use leads to social impairment and a tendency to withdraw from social interactions (Preller et al., 2014; Tomek et al., 2019). Furthermore, the HUD dyads displayed decreased IBS and brain activity during cooperation, providing neuroimaging evidence of social dysfunction in this population. These results confirm that individuals with HUD had deficits in cooperation during real-time turn-based interaction, and that such deficits may result from chronic heroin use impairing neural responses. Notably, compared to competitive interactions, HUD individuals showed significantly reduced IBS in the OFC, PFC, AG, and SAC during cooperation, and this reduction was strongly correlated with behavioural performance. These cortical regions are known to play critical roles in human cooperative behaviour (Zhao et al., 2024).
Consistent with previous studies (Lu et al., 2019; Zhao et al., 2022), network analysis revealed that cooperative performance was strongly associated with the increment of IBS in the AG, highlighting the critical role of IBS in the right angular gyrus (r-AG) during cooperative interactions. The AG is a key region within the Theory of Mind (ToM) network, with evidence indicating its involvement in integrating social information and interpreting the behavior of others (Schurz et al., 2017). AG dysfunction has been linked to ToM deficits across various psychiatric disorders (Su et al., 2016). Reduced IBS in the AG may reflect underlying ToM deficits, which could contribute to difficulties in cooperative tasks and broader social interactions. Consistent with previous studies, AG dysfunction has been shown to result in impaired mentalizing abilities during cooperation, reduced acquisition and perception of information about others, and deficits in spatial synergies required for task performance (Lotter et al., 2023; Luo et al., 2020). Our study further confirmed that AG was closely associated with heroin craving. Importantly, mediation analysis confirmed that heroin craving among individuals with HUD impaired cooperative performance by reducing IBS within the AG. This mediating effect remained marginally significant after controlling for years of heroin use and abstinence duration, suggesting that the observed mechanism is relatively robust and not simply confounded by individual differences in drug use history. These results identify a potential target for intervention in drug treatment and social rehabilitation. In the future, non-invasive approaches could be employed to further elucidate the role of IBS in the AG in regulating craving and cooperative performance (Wang et al., 2023; Esse Wilson et al., 2018; Wang et al., 2025). These findings offer mechanistic insights that may promote the development of precision interventions targeting social rehabilitation in individuals with HUD.
HUD participants exhibited reduced activation in the FPC under the cooperative condition, and this reduction was strongly correlated with impaired cooperative behavioural performance. Network analysis further identified FPC activation as the most central variable, suggesting its potential clinical significance in individuals with HUD. This finding aligns with previous studies demonstrating heightened FPC activity during the drug craving state in individuals with heroin, methamphetamine, and mixed drug use addiction (Yang et al., 2022). Such patterns may reflect a neuroadaptive shift induced by chronic drug use, increasing sensitivity to drug-related cues while blunting responsiveness to social interactions, as evidenced by altered FPC activation. Critically, as a key region within the PFC, the FPC regulates social reward circuits and orchestrates higher cognitive functions—including decision-making, executive, and attentional functions, which are critical for human social interactions, especially cooperative behaviors (Gläscher et al., 2012). The present study corroborated that chronic heroin use leads to structural and functional impairments in the PFC (King et al., 2022; Zhang et al., 2016), mirroring PFC dysfunction observed in cocaine use disorder (Ceceli et al., 2022; Preller et al., 2014). This PFC dysfunction was developed during chronic heroin use, leading to disruptions in neurotransmitter delivery, including dopamine, serotonin, and corticotropin-releasing factor (King et al., 2022; Wang et al., 2025). These neurotransmitters play a central role in regulating mood, motivation, and social behavior. Their absence makes it difficult for individuals with HUD to feel the pleasure of cooperation, which further diminishes their intrinsic drive to engage in social cooperation and exacerbates deficits in cooperative performance.
Previous studies have demonstrated that healthy individuals exhibit stronger brain activation and increased IBS during cooperative tasks than competitive ones (Zhao et al., 2025). HUD participants displayed blunted neurological sensitivity to social rewards resulting from long-term heroin use. This impairment manifested as diminished neural responses and reduced emotional resonance during social interaction, ultimately contributing to decreased tendency to cooperate (Yang et al., 2022). Specifically, it indicates that individuals with HUD are likely to encounter communication barriers in social interactions following withdrawal. Such impairments could hinder their ability to establish meaningful cooperative relationships, thereby potentially compromising their social rehabilitation efforts.
Preferential engagement in competition over cooperationWhile no significances were observed in IBS or individual brain activity between the HUD and healthy controls under competitive conditions, divergent patterns emerged in cooperation and competition within each group. These divergent patterns were manifested as follows: the neural responses were higher or no different under the cooperative condition than the competitive one in HC, but the competitive condition elicited higher responses than the cooperative one in HUD. Specifically, during competition, HUD participants exhibited higher IBS in the SMG (within the r-TPJ, a region associated with attentional processes and spatial cognitive functions) compared to cooperation. Typically, according to the shared intention hypothesis of inter-brain synchronization, a common goal often induces high IBS (Fishburn et al., 2018; Liu et al., 2023). Therefore, the HCs often display increased IBS in SMG during the cooperation task (Yin et al., 2025). However, in HUD participants, pursuing a destructive goal during competition appeared to generate stronger shared intentionality than engaging in a collaborative goal during cooperation. In other words, their objective was to "destroy" together rather than to "collaborate". These results may suggest a tendency among HUD participants to preferentially engage in competition. This phenomenon warrants further attention.
The OFC is typically activated during intoxication, craving, and substance use, and conversely deactivated during withdrawal (Uhl et al., 2019). Thus, the higher OFC activation observed in HUD participants during competition may imply that competitive contexts elicit a greater expectation or experience of reward. Considering the critical function of the OFC in addiction and its heightened sensitivity to reward stimuli, this elevated activation may further reinforce a preference for and tendency toward competition among individuals with HUD. This inclination may partly stem from a proself social value orientation, which prioritises individual interests over collective ones and thereby triggers stronger neural responses (Balconi & Vanutelli, 2017a; Zhao et al., 2025). These findings suggest that the HUD participants may display a distinct social motivation pattern, in which competitive contexts elicit stronger neural synchronization and activation than cooperative contexts, potentially reflecting altered social reward processing in this population.
Although individuals with HUD exhibited a significantly higher error rate during competitive interactions, this does not indicate weaker basic task competence, as no significant behavioral differences were observed between the HUD and healthy control groups under the independent condition. The poorer performance of HUD participants may instead be related to the intrinsic nature of competition and cooperation as socially demanding activities, both of which involve complex interpersonal interactions and require higher-order cognitive abilities, such as monitoring and mentalizing (Balconi & Vanutelli, 2017b). Although the HUD participants may have invested more effort in competition, this effort did not translate into better performance compared to the healthy controls due to their limitations in cognitive functioning. This may further reflect a tendency towards hyper-mentalizing under competitive conditions, resulting in cognitive overload and decision-making conflicts that undermine their behavioral efficiency (Alon et al., 2024). Furthermore, consistent with the neural response pattern, HUD participants exhibited significantly lower error rates under the competitive condition compared to their performance under the cooperative condition.
More critically, this dysfunctional preferential engagement in competition over cooperation may generalize to real-world social dysfunction, including interpersonal aggression, poor occupational collaboration, and maladaptive risk-taking behaviors. In clinical and rehabilitation settings, maladaptive competitive orientation undermines therapeutic alliances through disrupting peer support in group therapy via distrust, and triggers high-risk confrontations in social rehabilitation settings. Gradually, this cognitive and behavioral pattern in individuals with HUD is likely to exacerbate social alienation, thereby contributing to social stability risks and public health burdens. Ultimately, this would significantly increase relapse, placing an additional burden on the judicial administration. The detrimental effects of this maladaptive competitive orientation thus warrant particular clinical attention, given its implications for individual rehabilitation and broader societal stabilization.
LimitationsDespite revealing r-TPJ dysfunction as a mediator of heroin craving in impairing cooperative performance in individuals with HUD, our cross-sectional design precludes causal inference and highlights several additional limitations. First, the participants' selection was limited to individuals with HUD, which restricts the generalizability of the findings and warrants caution when attempting to apply these results to other kinds of drugs. Later studies could consider including individuals with diverse patterns of substance use to more comprehensively examine the detrimental effects of addiction on social interactions. Second, our study used a cross-sectional design and lacked a follow-up observation of changes in the patterns of cooperation and competition among participants with HUD throughout the withdrawal process, nor an evaluation of their long-term social functioning following reintegration into society. Future research could conduct a longitudinal follow-up study to explore the dynamics of the effects of chronic heroin use on social interactions over time. Third, the selection of IBS at CH20 as the mediator in this study's mediation model was initially identified through multiple channel-wise comparisons and correlation analyses. Although this 'screen-then-model' research approach has some validity and is widely used in exploratory neural mechanism studies (De Felice et al., 2025; Wei et al., 2023; Zhao et al., 2022), it is inherently post-hoc and may introduce selection bias. Therefore, these findings should be considered preliminary, and future studies using independent samples are needed to conduct confirmatory tests of the mediating effect identified here. Additionally, although standardized instructions and practice sessions were employed to ensure participants understood the task requirements, the absence of a formal manipulation check to quantitatively verify participants' perceived interpersonal goals represents a limitation. Future studies could incorporate explicit manipulation checks to further validate the experimental manipulation of social contexts and employ diverse cooperation-competition paradigms to further validate and extend the conclusions drawn from the present study. Finally, although the present study identified potential brain regions and neural mechanisms underlying social dysfunction in HUD, it did not directly address causal mechanisms. To this end, future studies may consider incorporating interventions such as electrical stimulation to provide a more robust theoretical foundation and empirical evidence to inform drug rehabilitation practices, thereby advancing the development of research in this field.
ConclusionIn conclusion, the present study elucidated the cognitive-neural mechanisms underlying cooperative and competitive response patterns in individuals with HUD during turn-based interactions. The results revealed abnormal behavioural and neural responses among HUD participants compared to healthy controls. Evidence from inter-brain neural synchrony and individual brain activation confirmed impaired cooperative performance and heightened competitive tendency in this population. Notably, the findings further demonstrated that heroin craving negatively affected cooperative performance by reducing IBS in the r-TPJ. Collectively, these results not only advance our understanding of the neural substrates of social dysfunction in individuals with HUD but also identify clinically relevant potential biomarkers that may inform the development of targeted neuromodulation interventions to facilitate social rehabilitation in HUD.
Author contributionsWanyi Li: Data curation, Formal analysis, Investigation, Methodology, Software, Visualization, Writing—original draft, Writing—review & editing. Yifan Wang: Conceptualization, Formal analysis, Investigation, Methodology, Project administration, Software, Validation, Writing—review & editing. Wenjuan Fu: Data curation, Investigation, Resources, Writing – review & editing. Jiaqi Dang: Investigation, Writing – review & editing. Yujia Meng: Writing – review & editing. Xinyang Xu: Investigation. Cunfeng Yuan: Project administration. Yadan Li: Methodology, Supervision, Writing—review & editing. Haijun Duan: Conceptualization, Funding acquisition, Project administration, Resources, Supervision, Writing – review & editing.
Data and code availability statementThe datasets and research materials are available from the corresponding author on reasonable request.
The authors declare that they have no known competing financial interests or personal relationships that could have appeared to influence the work reported in this paper.
This study was funded by the National Natural Science Foundation of China grant (32471114), the Advantage Education and Rehabilitation Programme for drug addiction from the Ministry of Justice (SFBJYJZXM2023-21-06), the Fundamental Research Funds for the Central Universities (GK202502005), the Special Support Program for Innovation Teams Led by High-level SanQin Talents of Shaanxi Province, the Research Program Fund for the Youth Innovation Team of Shaanxi Universities (2022SXSJZW105), the Research Program Fund for Key Project of Teacher Development of Shaanxi Province (2023JSZ005), the Research Program Fund for Higher Education Reform of Shaanxi Province (23ZZ022), the Natural Science Basic Research Program of Shaanxi (2025JC-YBMS-208), the Social Science Fund Project of Shaanxi (No. 2024P004).